
Compound Monograph
Cordycepin
Cordycepin (3'-deoxyadenosine) is the signature nucleoside of Cordyceps militaris — a cytotoxic adenosine analogue behind most of cordyceps' preclinical anticancer and anti-inflammatory claims, but rapidly destroyed by adenosine deaminase, which cripples its oral bioavailability and has pushed drug development toward a prodrug (NUC-7738).

Sources · 3
Where Does It Come From?
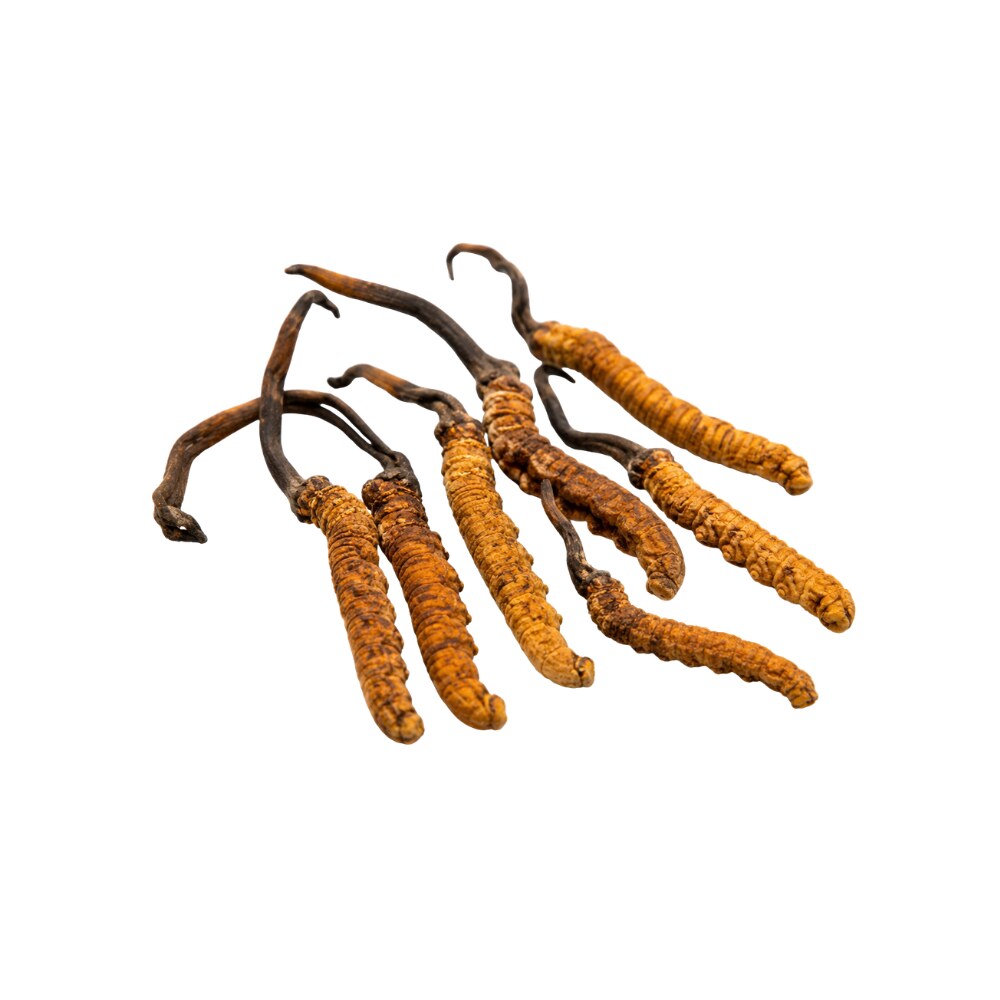
Cordycepin is a naturally occurring nucleoside analogue (3'-deoxyadenosine), found in Cordyceps militaris and 2 other sources. It is flagged as moderately toxic.
Concentration
Content by Source
Concentrations not reported. No percent-dry-weight or mg/g figures have been published for this compound in its source plants.
Cordycepin at a Glance
Cordycepin (3’-deoxyadenosine) is the signature nucleoside of Cordyceps militaris — an adenosine analogue missing a single hydroxyl group, which is enough to make it terminate RNA chains when incorporated.
That mechanism drives most of cordyceps’ preclinical anticancer and anti-inflammatory claims.
Its problem is the same missing group. Cordycepin is rapidly destroyed by adenosine deaminase in blood, which is why serious attempts to develop it pair it with a deaminase inhibitor — and why oral cordyceps products are unlikely to deliver meaningful systemic cordycepin.
What It's Used For
Cordycepin (3’-deoxyadenosine) is the signature nucleoside of Cordyceps militaris and the molecule behind most of cordyceps’ preclinical anticancer and anti-inflammatory reputation. Structurally it is adenosine missing its 3’-hydroxyl, and that single change defines both its mechanism and its problem. The mechanism: lacking a 3’-OH, it is incorporated into RNA as a chain terminator and blocks polyadenylation, disrupting RNA synthesis 4,
The problem: being a near-perfect adenosine mimic, it is rapidly deaminated by adenosine deaminase (ADA) to the largely inactive 3’-deoxyinosine, giving a minutes-scale half-life and poor oral bioavailability 9Reference 9AnimalSimultaneous determination of cordycepin and its metabolite 3’-deoxyinosine in rat whole blood by UHPLC-Q Exactive HRMS and application to pharmacokinetic studyView study →.
That liability has pushed drug development away from the molecule itself and toward a ProTide prodrug, NUC-7738, which is the source of the only human clinical data here 11Reference 11Clinical trialThe novel nucleoside-analogue ProTide NUC-7738 overcomes cancer resistance mechanisms in vitro and in a first-in-human Phase I clinical trialView study →.
Note up front: the “energy/stamina/libido” reputation belongs to whole cordyceps tradition, not to any isolated-cordycepin study.
Support is an experimental score — weighted by study type (human > animal > in vitro) and volume. A beta, not a validated metric. Isolated cordycepin is preclinical, so scores stay low by design. Each application links to its write-up.
The marquee application. Cordycepin is incorporated into RNA and terminates chain elongation and polyadenylation, induces apoptosis and cell-cycle arrest via AMPK activation 4Reference 4Cordycepin inhibits drug-resistant non-small-cell lung cancer progression by activating the AMPK signalling pathwayView study →, inhibits EGFR/ERK–Slug signaling in lung cancer 5Reference 5Cordycepin induces human lung cancer cell apoptosis by inhibiting nitric-oxide-mediated ERK/Slug signallingView study →, and reverses cisplatin resistance in non-small-cell lung cancer 4Reference 4Cordycepin inhibits drug-resistant non-small-cell lung cancer progression by activating the AMPK signalling pathwayView study →.
Gap: these effect sizes come from cell lines and mouse models; isolated cordycepin has essentially no human efficacy data, and the only clinical signal is from the ProTide prodrug NUC-7738 — not the molecule 11Reference 11Clinical trialThe novel nucleoside-analogue ProTide NUC-7738 overcomes cancer resistance mechanisms in vitro and in a first-in-human Phase I clinical trialView study →.
Cordycepin suppresses NF-κB via Akt/p38 in LPS-stimulated macrophages (lowering TNF-α, iNOS and COX-2) 1Reference 1Cordycepin inhibits lipopolysaccharide-induced inflammation by suppression of NF-κB through Akt and p38 inhibition in RAW 264.7 macrophage cellsView study →, drives M1→M2 macrophage repolarization limiting organ damage in septic mice 2Reference 2AnimalCordycepin induces M1/M2 macrophage polarization to attenuate liver and lung damage in immature septic mice via NF-κB/p65 inhibitionView study →, reduces pain and joint pathology in osteoarthritis rodents through its polyadenylation-inhibitor action 3Reference 3AnimalThe polyadenylation inhibitor cordycepin reduces pain, inflammation and joint pathology in rodent models of osteoarthritisView study →, and attenuates airway hyperreactivity in asthma models 8Reference 8AnimalCordycepin alleviates airway hyperreactivity in a murine model of asthma by attenuating the inflammatory processView study →.
Gap: consistent and mechanistically coherent, but entirely preclinical, with no human anti-inflammatory trial 1,
Cordycepin prevented hyperglycemia in alloxan-diabetic mice 6Reference 6AnimalCordycepin from Cordyceps militaris prevents hyperglycemia in alloxan-induced diabetic miceView study → and lowered serum lipids in hyperlipidemic hamsters and rats 7Reference 7AnimalLipid-lowering effect of cordycepin (3’-deoxyadenosine) from Cordyceps militaris on hyperlipidaemic hamsters and ratsView study →.
Gap: thin — roughly one study per endpoint, in chemically-induced models, with no dose-response in humans 6,
The chain-termination and polyadenylation-blockade mechanism gives a plausible broad antiviral rationale, historically studied against retroviral polyadenylation 12Reference 12Cordycepin: a bioactive metabolite with therapeutic potentialView study →.
Gap: dated and in-vitro only, confounded by the rapid ADA deactivation, with no modern controlled data — keep modest 12Reference 12Cordycepin: a bioactive metabolite with therapeutic potentialView study →.
Mechanisms
| Target / pathway | Effect | Relevant to |
|---|---|---|
| RNA polyadenylation / chain termination (incorporated as 3’-dATP; no 3’-OH) | truncates mRNA polyadenylation and transcription | anticanceranti-inflammatoryantiviral |
| AMPK activation | energy-stress signaling → apoptosis, growth arrest, resistance reversal | anticancer (NSCLC) |
| EGFR/ERK–Slug and NO signaling | ↓ proliferation, pro-apoptotic | anticancer (lung) |
| NF-κB via Akt/p38 inhibition | ↓ TNF-α, iNOS, COX-2, IL-1β/IL-6 | anti-inflammatorysepsisasthma |
| Adenosine A3 receptor (adenosine analogue) | receptor-mediated anti-inflammatory/signaling modulation | anti-inflammatory (reviewed) |
| mTOR (downstream of AMPK) | autophagy / growth-signal modulation | anticancer (supporting) |
Pharmacokinetics
The defining problem. Because cordycepin is a near-perfect adenosine mimic, it is rapidly deaminated by adenosine deaminase (ADA) to the largely inactive 3’-deoxyinosine, giving a very short plasma half-life — rat whole-blood work confirms cordycepin is consumed rapidly with 3’-deoxyinosine as the dominant circulating metabolite 9Reference 9AnimalSimultaneous determination of cordycepin and its metabolite 3’-deoxyinosine in rat whole blood by UHPLC-Q Exactive HRMS and application to pharmacokinetic studyView study →. Oral bioavailability of intact cordycepin is poor-to-negligible; one study argues the apparent oral effect may run through a “nucleoside rescue” route, where absorbed 3’-deoxyinosine is re-converted intracellularly to cordycepin triphosphate rather than intact cordycepin surviving first pass 10Reference 10A novel nucleoside rescue metabolic pathway may be responsible for the therapeutic effect of orally administered cordycepinView study →. Two workarounds define the field: co-administration with an ADA inhibitor (pentostatin) to keep cordycepin intact 12Reference 12Cordycepin: a bioactive metabolite with therapeutic potentialView study →, and the modern NUC-7738 ProTide prodrug, which bypasses ADA deamination and the rate-limiting first phosphorylation to deliver the active triphosphate intracellularly at far higher potency 11Reference 11Clinical trialThe novel nucleoside-analogue ProTide NUC-7738 overcomes cancer resistance mechanisms in vitro and in a first-in-human Phase I clinical trialView study →. The bottom line: intact-cordycepin systemic exposure from oral supplementation is low and fleeting, so efficacy figures from injected or ADA-protected preclinical work do not transfer to oral fruiting-body dosing.
Clinical trials
For isolated cordycepin there are no completed human efficacy trials. Human clinical data exist only for the prodrug NUC-7738, tested in the first-in-human NuTide:701 Phase I study in advanced solid tumors — reported well-tolerated with early signs of anticancer activity 11Reference 11Clinical trialThe novel nucleoside-analogue ProTide NUC-7738 overcomes cancer resistance mechanisms in vitro and in a first-in-human Phase I clinical trialView study →. This is a chemically distinct ProTide (much more potent than cordycepin in vitro), engineered specifically to overcome cordycepin’s ADA/pharmacokinetic liabilities, so it is evidence for the scaffold, not for taking cordycepin. Whole-herb cordyceps human trials exist but are not cordycepin-specific and belong to the herb page.
| Completed | Planned | Terminated | Preclinical |
|---|---|---|---|
| —(isolate); prodrug NUC-7738 Phase I | prodrug ongoing | — | Extensive |
Last checked: July 2026.
Toxicity & Safety
Cordycepin is an antiproliferative/cytotoxic nucleoside analogue — the same RNA-directed activity that makes it an anticancer candidate is intrinsically a genotoxic, antiproliferative liability rather than a benign “tonic” profile 4,
Dosage
There is no established or validated human oral dose for isolated cordycepin, and nothing here is a recommendation. Preclinical rodent studies typically use ~10–60 mg/kg (oral or intraperitoneal), often with ADA protection, which is not human-translatable. Supplements sell Cordyceps militaris extracts standardized to a stated cordycepin content, but purified cordycepin has no clinical dosing standard and its poor oral stability makes any oral figure unreliable. NUC-7738 (the prodrug, given intravenously on a trial-defined escalation) is a separate agent — its dosing is not a cordycepin dose 11Reference 11Clinical trialThe novel nucleoside-analogue ProTide NUC-7738 overcomes cancer resistance mechanisms in vitro and in a first-in-human Phase I clinical trialView study →.
References
- Kim HG, et al. (2006). Cordycepin inhibits lipopolysaccharide-induced inflammation by suppression of NF-κB through Akt and p38 inhibition in RAW 264.7 macrophage cells. European Journal of Pharmacology. https://pubmed.ncbi.nlm.nih.gov/16899239/
- Zhang Y, Cheng J, Su Y, et al. (2022). Cordycepin induces M1/M2 macrophage polarization to attenuate liver and lung damage in immature septic mice via NF-κB/p65 inhibition. Journal of Pharmacy and Pharmacology. https://pubmed.ncbi.nlm.nih.gov/34850068/
- Ashraf S, et al. (2019). The polyadenylation inhibitor cordycepin reduces pain, inflammation and joint pathology in rodent models of osteoarthritis. Scientific Reports. https://pubmed.ncbi.nlm.nih.gov/30886197/
- Wei C, et al. (2019). Cordycepin inhibits drug-resistant non-small-cell lung cancer progression by activating the AMPK signalling pathway. Pharmacological Research. https://pubmed.ncbi.nlm.nih.gov/30974169/
- Hwang JH, et al. (2017). Cordycepin induces human lung cancer cell apoptosis by inhibiting nitric-oxide-mediated ERK/Slug signalling. American Journal of Cancer Research. https://pubmed.ncbi.nlm.nih.gov/28401001/
- Ma L, et al. (2015). Cordycepin from Cordyceps militaris prevents hyperglycemia in alloxan-induced diabetic mice. Nutrition Research. https://pubmed.ncbi.nlm.nih.gov/25940982/
- Gao J, et al. (2011). Lipid-lowering effect of cordycepin (3’-deoxyadenosine) from Cordyceps militaris on hyperlipidaemic hamsters and rats. Yao Xue Xue Bao (Acta Pharmaceutica Sinica). https://pubmed.ncbi.nlm.nih.gov/21882527/
- Yang X, et al. (2015). Cordycepin alleviates airway hyperreactivity in a murine model of asthma by attenuating the inflammatory process. International Immunopharmacology. https://pubmed.ncbi.nlm.nih.gov/25912153/
- Qi C, et al. (2023). Simultaneous determination of cordycepin and its metabolite 3’-deoxyinosine in rat whole blood by UHPLC-Q Exactive HRMS and application to pharmacokinetic study. Journal of Separation Science. https://pubmed.ncbi.nlm.nih.gov/36377517/
- Lee JB, Radhi M, Cipolla E, et al. (2019). A novel nucleoside rescue metabolic pathway may be responsible for the therapeutic effect of orally administered cordycepin. Scientific Reports. https://pubmed.ncbi.nlm.nih.gov/31673018/
- Schwenzer H, et al. (2021). The novel nucleoside-analogue ProTide NUC-7738 overcomes cancer resistance mechanisms in vitro and in a first-in-human Phase I clinical trial. Clinical Cancer Research. https://pubmed.ncbi.nlm.nih.gov/34497073/
- Tuli HS, et al. (2013). Cordycepin: a bioactive metabolite with therapeutic potential. Life Sciences. https://pubmed.ncbi.nlm.nih.gov/24121015/



