
Compound Monograph
Thymohydroquinone
Thymohydroquinone is the reduced, hydroquinone half of the thymoquinone redox couple in black seed oil — a direct radical scavenger that beats thymoquinone in several head-to-head enzyme and antioxidant assays, but which has almost no evidence of its own outside the test tube.

Sources · 5
Where Does It Come From?
Thymohydroquinone is a naturally occurring monoterpenoid (monoterpene hydroquinone / benzene-1,4-diol), found in Nigella, Thyme and 3 other sources. It is flagged as moderately toxic.
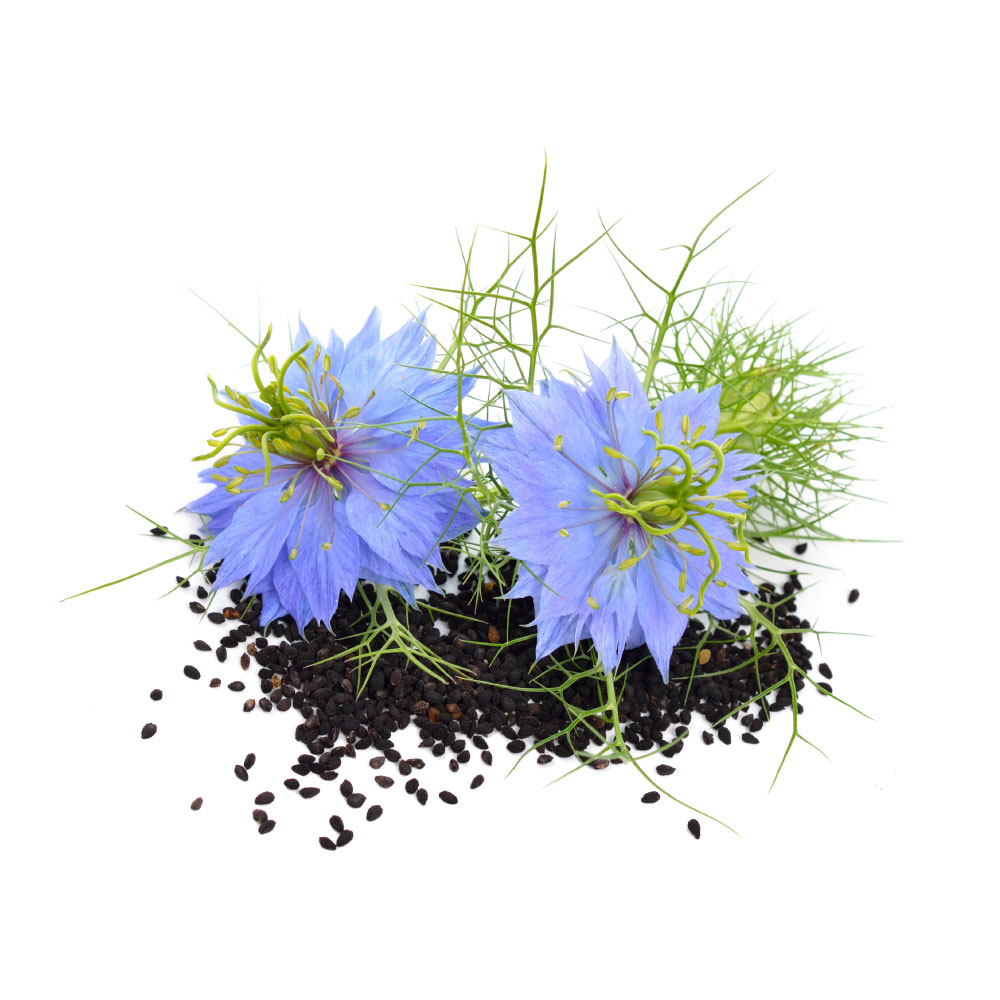 Principal source Nigella Nigella sativa Herb monograph →
Photo coming soon
Source Thyme Thymus vulgaris Herb monograph →
Concentration
Content by Source
Reported concentrations across the plants that contain thymohydroquinone — the bar marks the typical level, the line shows the reported range.
Literature figures for varying plant parts and preparations. Read them as a comparative guide, not exact assays.
Thymohydroquinone at a Glance
Thymohydroquinone (THQ) is the reduced form of thymoquinone — the same carbon skeleton with the two ring oxygens carrying hydrogens instead of sitting as a quinone. The two are not really independent compounds. They are two oxidation states of one system, interconverting in the seed oil on contact with air and inside cells through quinone reductases 7,
That relationship is the whole page. It has an immediate practical consequence: a published figure for either molecule is a snapshot of a redox equilibrium, not a fixed property of the plant. Extraction temperature, solvent, light exposure and how long the oil has sat all shift the ratio, which is why supercritical-CO₂ extracts recover a different quinone profile from hydrodistilled oil of the same seed 5Reference 5Chemical composition of Nigella sativa L. seed extracts obtained by supercritical carbon dioxideView study →.
The honest posture on the pharmacology is that the isolate literature here is thin — a few dozen papers, nearly all in vitro, no human trial, no pharmacokinetics. What makes it worth a page anyway is that the head-to-head assays are genuinely surprising: in several of them THQ is the more potent of the pair, not the inert one 7,
The Thymoquinone–Thymohydroquinone Redox Couple
Thymoquinone is a para-benzoquinone; thymohydroquinone is the corresponding hydroquinone. Add two electrons and two protons to the quinone and you get the diol; remove them and you get the quinone back. The couple runs in both directions in ordinary conditions:
- In the oil. Thymohydroquinone was first obtained precisely because it separates out of black-seed volatile oil on refrigeration 2Reference 2Isolation and structure assignment of an antimicrobial principle from the volatile oil of Nigella sativa L. seedsView study →, and the four quinonic phenols of the seed — thymoquinone, dithymoquinone, thymohydroquinone and thymol — are all thermally labile or photosensitive, so the measured ratio between them depends on the extraction route 5Reference 5Chemical composition of Nigella sativa L. seed extracts obtained by supercritical carbon dioxideView study →. Supercritical-CO₂ extraction recovers more of the phenolic set than hydrodistillation of the same material 5Reference 5Chemical composition of Nigella sativa L. seed extracts obtained by supercritical carbon dioxideView study →. An aged, warm, light-exposed oil is not chemically the same product as a fresh cold-pressed one.
- In the cell. Mammalian NAD(P)H:quinone oxidoreductase 1 (NQO1) performs the two-electron reduction of quinones to hydroquinones, and it does so to thymoquinone. In a panel of human breast-cancer lines, MCF-7 cells resisted thymoquinone’s cytotoxicity because they expressed high NQO1; blocking the enzyme with dicoumarol made them sensitive again 13Reference 13NADPH quinone oxidoreductase 1 mediates breast cancer cell resistance to thymoquinone-induced apoptosisView study →. In that setting, converting the quinone to the hydroquinone is a detoxification step.
- In microbes and in us. The traffic runs the other way too. Nocardia and Mycobacterium species hydroxylate thymol to thymohydroquinone and then oxidise it onward to thymoquinone 20Reference 20Two different primary oxidation mechanisms during biotransformation of thymol by gram-positive bacteria of the genera Nocardia and MycobacteriumView study →, and the same thymol → thymohydroquinone hydroxylation shows up as a minor pathway in human urine, where THQ appears to be excreted as a sulfate conjugate 19Reference 19On the metabolic detoxication of thymol in rabbit and manView study →.
The consequence for reading the literature is unglamorous but load-bearing: a “thymoquinone” result and a “thymohydroquinone” result may be describing the same molecular pool at different points on the same axis, and neither number tells you what fraction was in which state when the biology happened.
Is the Hydroquinone the Active Form?
The default assumption — that thymoquinone is the active one and the hydroquinone is its spent form — is not what the head-to-head data show. Where the two have been run side by side, the results split by assay type, and the split is informative.
| Property | Thymoquinone (TQ) | Thymohydroquinone (THQ) |
|---|---|---|
| DPPH radical scavenging (IC₅₀) | ~170 µg/mL (weak) 9Reference 9Determination of oxygen radical absorbance capacity of black cumin (Nigella sativa) seed quinone compoundsView study → | ~2.4 µg/mL (~70× stronger) 9Reference 9Determination of oxygen radical absorbance capacity of black cumin (Nigella sativa) seed quinone compoundsView study → |
| ORAC (Trolox equivalents) | 1.91 TE 9Reference 9Determination of oxygen radical absorbance capacity of black cumin (Nigella sativa) seed quinone compoundsView study → | 2.60 TE 9Reference 9Determination of oxygen radical absorbance capacity of black cumin (Nigella sativa) seed quinone compoundsView study → |
| Radical scavenging by ESR | weaker 7Reference 7Antioxidant and prooxidant effects of thymoquinone and its hydroquinone metaboliteView study → | stronger 7Reference 7Antioxidant and prooxidant effects of thymoquinone and its hydroquinone metaboliteView study → |
| Superoxide (O₂⁻) scavenging | active 8Reference 8Antioxidant properties of thymoquinone, thymohydroquinone and black cumin (Nigella sativa L.) seed oil: scavenging of superoxide radical studied using cyclic voltammetry, DFT and single crystal X-ray diffractionView study → | inactive 8Reference 8Antioxidant properties of thymoquinone, thymohydroquinone and black cumin (Nigella sativa L.) seed oil: scavenging of superoxide radical studied using cyclic voltammetry, DFT and single crystal X-ray diffractionView study → |
| COX-2 inhibition (IC₅₀) | 0.3 µM 14Reference 14In vitroIn vitro inhibitory effects of thymol and quinones of Nigella sativa seeds on cyclooxygenase-1- and -2-catalyzed prostaglandin E2 biosynthesesView study → | 0.1 µM 14Reference 14In vitroIn vitro inhibitory effects of thymol and quinones of Nigella sativa seeds on cyclooxygenase-1- and -2-catalyzed prostaglandin E2 biosynthesesView study → |
| 5-LOX / LTB₄ biosynthesis (IC₅₀) | 18.2 µM 15Reference 15In vitroInhibition of in vitro leukotriene B4 biosynthesis in human neutrophil granulocytes and docking studies of natural quinonesView study → | 4.1 µM 15Reference 15In vitroInhibition of in vitro leukotriene B4 biosynthesis in human neutrophil granulocytes and docking studies of natural quinonesView study → |
| Acetylcholinesterase inhibition | weaker than carvacrol 10Reference 10In vitroIn vitro acetylcholinesterase inhibitory properties of thymol, carvacrol and their derivatives thymoquinone and thymohydroquinoneView study → | strongest of the series tested 10Reference 10In vitroIn vitro acetylcholinesterase inhibitory properties of thymol, carvacrol and their derivatives thymoquinone and thymohydroquinoneView study → |
| Cytotoxicity to tumour cell lines | significant, dose-dependent 12Reference 12In vitroThe antitumor activity of thymoquinone and thymohydroquinone in vitro and in vivoView study → | significant, dose-dependent 12Reference 12In vitroThe antitumor activity of thymoquinone and thymohydroquinone in vitro and in vivoView study → |
| Cellular NQO1 expression | confers resistance to TQ 13Reference 13NADPH quinone oxidoreductase 1 mediates breast cancer cell resistance to thymoquinone-induced apoptosisView study → | (the product of that reduction) |
Three readings are defensible, and the evidence does not yet choose between them:
- THQ is the better direct antioxidant, and TQ is the better electrophile. This is the cleanest structural story. A hydroquinone has two donatable phenolic hydrogens, so it quenches radicals directly — hence the ~70-fold DPPH advantage and the stronger ESR signal 7,
9Reference 7Antioxidant and prooxidant effects of thymoquinone and its hydroquinone metaboliteView study →Reference 9Determination of oxygen radical absorbance capacity of black cumin (Nigella sativa) seed quinone compoundsView study → . A quinone has none; thymoquinone’s antioxidant reputation rests instead on being an electrophile that reacts with thiols and switches on Nrf2/ARE-driven cytoprotective genes, an indirect route 8,13Reference 8Antioxidant properties of thymoquinone, thymohydroquinone and black cumin (Nigella sativa L.) seed oil: scavenging of superoxide radical studied using cyclic voltammetry, DFT and single crystal X-ray diffractionView study →Reference 13NADPH quinone oxidoreductase 1 mediates breast cancer cell resistance to thymoquinone-induced apoptosisView study → . The two molecules are antioxidants by different mechanisms, which is why they rank differently depending on which assay you pick. Superoxide is the giveaway: thymoquinone scavenges it via a quinone–superoxide radical adduct that thymohydroquinone simply cannot form, so on that specific radical the ordering inverts 8Reference 8Antioxidant properties of thymoquinone, thymohydroquinone and black cumin (Nigella sativa L.) seed oil: scavenging of superoxide radical studied using cyclic voltammetry, DFT and single crystal X-ray diffractionView study →. - THQ is the inactivated form. The NQO1 result supports this in at least one context — reduction to the hydroquinone is what lets a cancer cell survive thymoquinone 13Reference 13NADPH quinone oxidoreductase 1 mediates breast cancer cell resistance to thymoquinone-induced apoptosisView study →.
- THQ is a reservoir. Neither of the above excludes the couple acting as a redox buffer, with the hydroquinone re-oxidising to regenerate the electrophile. Nobody has measured this in a tissue, and that is the honest state of the question.
What can be said flatly: the assumption that the hydroquinone is the inert one is not supported. In four separate direct-target assays — COX-2, 5-LOX, acetylcholinesterase and DPPH — thymohydroquinone was the stronger of the two 9,
What It's Used For
The whole file is preclinical. There is no human trial of thymohydroquinone, no pharmacokinetic study, and no dose-ranging work; what exists is a scattered set of in-vitro enzyme, radical and microbiology assays plus one small mouse tumour experiment.
Support is an experimental score — weighted by study type (human > animal > in vitro) and volume. A beta, not a validated metric. Every row here is capped low for the same reason: there is no human evidence for this isolate at all, so read these as relative strength within a preclinical file.
The best-characterised property, and the one where the isolate — not an extract — was actually tested. Against DPPH, thymohydroquinone gave an IC₅₀ of 2.4 µg/mL versus thymoquinone’s 170 µg/mL, and it scored 2.60 Trolox equivalents in ORAC against thymoquinone’s 1.91; dithymoquinone was inactive 9Reference 9Determination of oxygen radical absorbance capacity of black cumin (Nigella sativa) seed quinone compoundsView study →.
Electron-spin-resonance work independently found THQ the more potent antioxidant of the pair 7Reference 7Antioxidant and prooxidant effects of thymoquinone and its hydroquinone metaboliteView study →.
The important counter-result: using a direct electrochemical (rotating ring-disk) method with DFT support, thymoquinone and whole black-seed oil scavenged superoxide while thymohydroquinone did not — the mechanism there requires formation of a quinone–superoxide radical adduct that a hydroquinone cannot make 8Reference 8Antioxidant properties of thymoquinone, thymohydroquinone and black cumin (Nigella sativa L.) seed oil: scavenging of superoxide radical studied using cyclic voltammetry, DFT and single crystal X-ray diffractionView study →.
So “antioxidant” is radical-specific, not a general ranking.
Gap: all of it is chemistry-bench assay data on the pure compound. No cellular antioxidant-response, animal oxidative-stress model or human biomarker study exists for thymohydroquinone, and the same paper that found it the better antioxidant also found it a prooxidant in the presence of free transition metals 7Reference 7Antioxidant and prooxidant effects of thymoquinone and its hydroquinone metaboliteView study →.
Two isolate studies from overlapping Czech groups give thymohydroquinone the strongest numbers in this file. Against cyclooxygenase-catalysed prostaglandin-E₂ biosynthesis, THQ was the most active of the black-seed quinones on COX-2 (IC₅₀ 0.1 µM), ahead of thymoquinone (0.3 µM), with thymol leading on COX-1 (0.2 µM) — all at concentrations comparable to indomethacin 14Reference 14In vitroIn vitro inhibitory effects of thymol and quinones of Nigella sativa seeds on cyclooxygenase-1- and -2-catalyzed prostaglandin E2 biosynthesesView study →.
In activated human neutrophil granulocytes, THQ inhibited leukotriene-B₄ biosynthesis at IC₅₀ 4.1 µM, matching the reference 5-LOX inhibitor zileuton (4.1 µM) and beating thymoquinone (18.2 µM); molecular docking suggested that for 5-LOX the molecular structure, not simply redox potential, drives the activity 15Reference 15In vitroInhibition of in vitro leukotriene B4 biosynthesis in human neutrophil granulocytes and docking studies of natural quinonesView study →.
Dual COX-2/5-LOX activity in the same molecule is a real pharmacological point of interest.
Gap: cell-free enzyme and isolated-neutrophil assays only. There is no animal inflammation model and no human study of thymohydroquinone, and no data on whether the free compound ever reaches an inflamed tissue at 0.1–4 µM after oral black-seed oil.
Thymohydroquinone entered the literature as an antimicrobial: the crystalline substance that separates out of refrigerated Nigella sativa volatile oil was identified in 1975 as thymohydroquinone and reported to have high activity against gram-positive organisms 2Reference 2Isolation and structure assignment of an antimicrobial principle from the volatile oil of Nigella sativa L. seedsView study →.
Modern quantification is modest but real — against six dairy-spoilage yeast species, THQ and thymoquinone both inhibited every strain at MICs of 8–128 µg/mL, and, unlike calcium propionate and potassium sorbate, their activity held up across pH 4.0 and 5.5 16Reference 16In vitroIn vitro antifungal effect of black cumin seed quinones against dairy spoilage yeasts at different acidity levelsView study →.
More recently, thymohydroquinone was one of six phytochemicals that reduced biofilm formation and downregulated biofilm-linked and antimicrobial-resistance genes in wastewater Aeromonas isolates 18Reference 18Natural compound-induced downregulation of antimicrobial resistance and biofilm-linked genes in wastewater Aeromonas speciesView study →.
In Zataria multiflora, thymohydroquinone glycoconjugates correlated with antifungal activity of leaf extracts, though bioassay-guided fractionation ultimately pointed at methylated flavones rather than the THQ conjugates 21Reference 21Metabolite profiling and bioassay-guided fractionation of Zataria multiflora Boiss. hydroethanolic leaf extracts for identification of broad-spectrum pre- and postharvest antifungal agentsView study →.
Gap: all in vitro, and mostly food-microbiology or environmental rather than clinical organisms. The MICs (8–128 µg/mL) are far above anything plausibly achievable systemically, so this is a preservative/topical-scale activity, not evidence of an oral anti-infective.
One study has tested the pair head to head in vivo. Thymoquinone and thymohydroquinone were both significantly cytotoxic (p ≤ 0.01) to squamous-cell-carcinoma and fibrosarcoma lines and more so to tumour cells than to L929 fibroblasts; in two murine tumour models, four intratumoral injections at 5 mg/kg produced tumour-growth inhibition of 52%, and the authors concluded THQ’s effect might improve at higher doses 12Reference 12In vitroThe antitumor activity of thymoquinone and thymohydroquinone in vitro and in vivoView study →.
The redox context matters here more than the raw numbers: high tumour NQO1 expression protects breast-cancer cells from thymoquinone precisely by reducing it, which implies the quinone — not the hydroquinone — is the cytotoxic species in that cell type 13Reference 13NADPH quinone oxidoreductase 1 mediates breast cancer cell resistance to thymoquinone-induced apoptosisView study →.
Gap: a single small 2006 animal study using intratumoral injection, a route that says nothing about oral or systemic use, and no replication in twenty years. The apparent tumour selectivity is from crystal-violet viability assays, not a therapeutic index.
Testing the constituents of Thymus vulgaris essential oil, thymohydroquinone showed the strongest acetylcholinesterase inhibition across the concentration range, with the order running THQ > carvacrol > thymoquinone > whole essential oil > thymol > linalool 10Reference 10In vitroIn vitro acetylcholinesterase inhibitory properties of thymol, carvacrol and their derivatives thymoquinone and thymohydroquinoneView study →.
A later review of essential-oil constituents as cholinesterase inhibitors lists thymohydroquinone among the notably active compounds 11Reference 11Terpenes, phenylpropanoids, sulfur and other essential oil constituents as inhibitors of cholinesterasesView study →.
A separate in-silico study docked THQ against blood–brain-barrier-disrupting proteins and predicted CNS permeability — while simultaneously predicting high acute toxicity 22Reference 22In silico study of thymohydroquinone interaction with blood-brain barrier disrupting proteinsView study →.
Gap: a single in-vitro enzyme series from 2007 with no IC₅₀ reported in the abstract, one review echoing it, and one docking paper. There is no cellular, animal or cognitive data, and docking-derived “BBB permeant” claims are hypotheses, not measurements.
Thymohydroquinone and dithymoquinone, both prepared semi-synthetically from thymoquinone, were tested against SARS-CoV-2 in vitro. Activity appeared at non-cytotoxic nanomolar concentrations but with a selectivity index of only 1.4 (CC₅₀ 31.74 / IC₅₀ 23.15), with dithymoquinone the more cytotoxic of the two 17Reference 17In vitroIn vitro potential antiviral SARS-CoV-19 activity of natural product thymohydroquinone and dithymoquinone from Nigella sativaView study →. A selectivity index that close to 1 means the antiviral and toxic concentrations essentially overlap.
Gap: one cell-culture study, on semi-synthetic rather than plant-isolated material, with a selectivity index too narrow to be of therapeutic interest. Every other “Nigella against COVID” paper in this space is molecular docking. No animal or human antiviral data exist.
Mechanisms
| Target / pathway | Effect | Relevant to |
|---|---|---|
| Direct hydrogen-atom donation (two phenolic OH) | quenches DPPH and other radicals directly — ~70× thymoquinone’s DPPH potency | antioxidant (the structural signature of a hydroquinone) |
| Superoxide (O₂⁻) | no scavenging — the quinone–superoxide adduct route is unavailable to a hydroquinone | the clearest mechanistic split from thymoquinone |
| Transition-metal redox cycling (free Cu²⁺, Fe²⁺–EDTA) | prooxidant: oxidative damage to isolated plasmid DNA | toxicity / the flip side of redox activity |
| COX-2 | inhibition of prostaglandin-E₂ biosynthesis, IC₅₀ 0.1 µM (cell-free) | anti-inflammatory |
| 5-Lipoxygenase / LTB₄ | inhibition at IC₅₀ 4.1 µM in human neutrophils; structure-driven binding, not purely redox | anti-inflammatory |
| Acetylcholinesterase | inhibition; ranked first among thyme-oil constituents tested | cholinergic / neuro (hypothetical) |
| NQO1 (NAD(P)H:quinone oxidoreductase 1) | THQ is the product of NQO1 reduction of thymoquinone; high NQO1 confers thymoquinone resistance | the redox couple; cancer-cell pharmacology |
| Microbial membranes / biofilm gene expression | growth inhibition of yeasts (MIC 8–128 µg/mL); downregulation of biofilm and resistance genes | antimicrobial |
The load-bearing contrast: thymoquinone works largely as an electrophile — reacting with thiols and switching on Nrf2/ARE cytoprotection — whereas thymohydroquinone works as a direct hydrogen donor. Calling both “antioxidants” hides the fact that they get there by opposite chemistry, and it is why their rank order flips between assays 7,
Pharmacokinetics
There are none. No absorption, distribution, metabolism, excretion, bioavailability, Cmax or half-life figures have been published for thymohydroquinone in any species. This is the single largest hole on the page, and it undercuts every in-vitro number above: the COX-2 IC₅₀ of 0.1 µM and the 5-LOX IC₅₀ of 4.1 µM are meaningless as therapeutic claims until somebody shows the free compound reaches those concentrations somewhere in a body.
What little is known is metabolic rather than kinetic, and points the other way — toward thymohydroquinone as an intermediate rather than a circulating agent. In humans given thymol, thymohydroquinone appears in urine only in small amounts and appears to be excreted as a sulfate conjugate 19Reference 19On the metabolic detoxication of thymol in rabbit and manView study → — the same rapid phase-II conjugation that keeps free thymol out of the circulation. Bacteria that metabolise thymol pass through thymohydroquinone transiently and then oxidise it onward to thymoquinone 20Reference 20Two different primary oxidation mechanisms during biotransformation of thymol by gram-positive bacteria of the genera Nocardia and MycobacteriumView study →, and fungal systems glucosylate it 23Reference 23Microbial models of mammalian metabolismView study →. All of that is consistent with a molecule that is conjugated or re-oxidised quickly rather than one that persists free in plasma.
Clinical Trials
None. No clinical trial of isolated thymohydroquinone has been registered or reported; human evidence in this area belongs to whole Nigella sativa seed or oil, where thymohydroquinone is a minor constituent among many and was never the variable under test 25Reference 25Pharmacological and toxicological properties of Nigella sativaView study →.
| Completed | Planned | Terminated | Preclinical |
|---|---|---|---|
| — | — | — | In-vitro antioxidant, COX-2/5-LOX, antimicrobial, cytotoxicity; one mouse intratumoral study |
Last checked: July 2026.
Isolate vs. Plant Studies
Unusually, this molecule’s problem is the reverse of the usual one. The preclinical work here mostly does use the purified isolate — the DPPH/ORAC comparison, the ESR study, the COX and 5-LOX assays, the yeast MICs and the mouse tumour experiment all tested pure thymohydroquinone, often side by side with pure thymoquinone 7,
The failure mode is transfer in the other direction: taking the large human and animal record built on Nigella sativa oil, or on thymoquinone, and applying it to this molecule. That record is not thymohydroquinone’s. Black-seed oil trials measure an oil in which THQ is roughly a tenth as abundant as thymoquinone 4Reference 4In vitroComposition, in vitro antioxidant and antimicrobial activities of essential oil and oleoresins obtained from black cumin seeds (Nigella sativa L.)View study →; the antidiabetic, lipid and anti-inflammatory human signals attributed to the seed are attributed, in the source literature, to the whole preparation or to thymoquinone 25Reference 25Pharmacological and toxicological properties of Nigella sativaView study →. Nothing here should be read as evidence that taking black seed oil delivers a pharmacologically active dose of thymohydroquinone, and nothing in thymoquinone’s file should be silently inherited here.
Its Role in Plants
Thymohydroquinone sits at the end of the phenolic-monoterpene branch of the Lamiaceae/Ranunculaceae volatile pathway. Geranyl diphosphate is cyclised to γ-terpinene, which cytochrome P450s of the CYP71D subfamily oxidise to unstable cyclohexadienol intermediates; a short-chain dehydrogenase/reductase then converts these to the corresponding ketones, which tautomerise to the aromatic phenols thymol and carvacrol — with p-cymene forming instead when the dehydrogenase is absent. Two further P450s, of the CYP76S and CYP736A subfamilies, then hydroxylate thymol and carvacrol to thymohydroquinone 6Reference 6The biosynthesis of thymol, carvacrol, and thymohydroquinone in Lamiaceae proceeds via cytochrome P450s and a short-chain dehydrogenaseView study →. So THQ is not a degradation product; it is an enzymatically produced end-point, one oxidation step past the plant’s better-known phenols.
In Nigella sativa the compound has a defined location and timing. Seed volatiles are dominated by p-cymene, thymohydroquinone, thymoquinone, γ-terpinene and α-thujene, and these — along with the indazole alkaloids nigellidine and nigellicine — accumulate almost exclusively in the seed coat, while organic and amino acids sit in the inner tissues 3Reference 3Distribution of primary and specialized metabolites in Nigella sativa seeds, a spice with vast traditional and historical usesView study →. The profile also changes as the seed matures: γ-terpinene and α-thujene dominate immature seed, and γ-terpinene is progressively replaced by p-cymene, carvacrol, thymohydroquinone and thymoquinone as the seed develops 3Reference 3Distribution of primary and specialized metabolites in Nigella sativa seeds, a spice with vast traditional and historical usesView study →. A seed-coat localisation of an antimicrobial, redox-active phenol is a textbook chemical-defence arrangement, though the ecological function has not been tested directly.
Prevalence in Nature
Thymohydroquinone is a minor but consistent member of the black-seed quinone set. GC-MS of Nigella sativa seed essential oil put it at 3.4% of the oil, behind thymoquinone (37.6%), p-cymene (31.2%) and α-thujene (5.6%) 4Reference 4In vitroComposition, in vitro antioxidant and antimicrobial activities of essential oil and oleoresins obtained from black cumin seeds (Nigella sativa L.)View study →; an HPLC method for the four pharmacologically relevant compounds of the seed oil — thymoquinone, dithymoquinone, thymohydroquinone and thymol — established it as a routine quality-control analyte 1Reference 1High performance liquid chromatographic analysis of the pharmacologically active quinones and related compounds in the oil of the black seed (Nigella sativa L.)View study →. Because all four are thermally labile or photosensitive, the numbers are method-bound: supercritical-CO₂ extraction recovers the phenolic set better than hydrodistillation from the same seed 5Reference 5Chemical composition of Nigella sativa L. seed extracts obtained by supercritical carbon dioxideView study →. Whole-seed figures should be treated with more caution still, given how variable Nigella’s quinone content is with origin, storage and processing 25Reference 25Pharmacological and toxicological properties of Nigella sativaView study →.
Beyond Nigella, the compound belongs to the Lamiaceae phenolic-monoterpene chemotypes, since the enzymes that make it act on thymol and carvacrol 6Reference 6The biosynthesis of thymol, carvacrol, and thymohydroquinone in Lamiaceae proceeds via cytochrome P450s and a short-chain dehydrogenaseView study → — it is described as a constituent among the derivatives of Thymus vulgaris oil 10Reference 10In vitroIn vitro acetylcholinesterase inhibitory properties of thymol, carvacrol and their derivatives thymoquinone and thymohydroquinoneView study →, and in Iranian Shirazi thyme (Zataria multiflora) it occurs as a set of thymohydroquinone glycoconjugates rather than the free phenol 21Reference 21Metabolite profiling and bioassay-guided fractionation of Zataria multiflora Boiss. hydroethanolic leaf extracts for identification of broad-spectrum pre- and postharvest antifungal agentsView study →. It is also, marginally, a human metabolite: people given thymol excrete small amounts of thymohydroquinone, apparently as a sulfate conjugate 19Reference 19On the metabolic detoxication of thymol in rabbit and manView study →, and thymol-degrading bacteria and fungi generate it as an intermediate 20,
A Note on Thymohydroquinone Dimethyl Ether
A large share of what a literature search returns for “thymohydroquinone” is actually about thymohydroquinone dimethyl ether — a different compound, in which both hydroxyls are methylated. It is the main constituent of Ayapana triplinervis essential oil and carries its own literature on Zika-virus inhibition in zebrafish, antinociception and Aedes larvicide 24Reference 24Ayapana triplinervis essential oil and its main component thymohydroquinone dimethyl ether inhibit Zika virus at doses devoid of toxicity in zebrafishView study →.
The distinction is not pedantic. Methylating both hydroxyls removes exactly the feature at issue — the donatable phenolic hydrogens that make a hydroquinone a direct radical scavenger, and the ability to be oxidised back to the quinone. The dimethyl ether cannot participate in the thymoquinone redox couple at all. None of its activity data transfer to thymohydroquinone, and none appear here.
Discovery & Synthesis
First isolation. Thymohydroquinone was obtained as a natural product from black seed by a simple physical trick: refrigerating the volatile oil of Nigella sativa seeds causes a crystalline substance to separate, and in 1975 El-Fatatry assigned its structure — from chemical behaviour plus UV, IR, PMR and mass spectra, confirmed via the diacetate ester — as thymohydroquinone, reporting high activity against gram-positive organisms 2Reference 2Isolation and structure assignment of an antimicrobial principle from the volatile oil of Nigella sativa L. seedsView study →. The molecule was known to chemistry before that as an oxidation product of thymol; a laboratory synthesis was published by Svishchuk and Visotskii in 1970 26Reference 26Svishchuk OA, Visotskii MM (1970). [Synthesis of thymohydroquinone]. Farmatsevtychnyi Zhurnal. https://pubmed.ncbi.nlm.nih.gov/5505177/View study →, and an improved synthetic protocol was later developed explicitly to make the compound more available for research 9Reference 9Determination of oxygen radical absorbance capacity of black cumin (Nigella sativa) seed quinone compoundsView study →. Earlier still, thymoquinone and thymohydroquinone were being compared against the classical uncoupler 2,4-dinitrophenol in yeast-metabolism experiments in 1960 27Reference 27Flaig W, de Jong (1960). [Comparison of the effect of thymoquinone and thymohydroquinone with that of 2,4-dinitrophenol on the metabolism of yeasts (Saccharomyces cerevisiae)]. Archiv für Mikrobiologie. https://pubmed.ncbi.nlm.nih.gov/13700109/View study →, which places the pair in the biochemical literature well before the modern Nigella interest.
Manufacture today. There is no commercial extraction industry for thymohydroquinone. Research material is synthetic or semi-synthetic — typically prepared by reduction of thymoquinone or oxidation of thymol, the same two-step relationship the molecule has in nature; the SARS-CoV-2 study, for instance, used THQ and dithymoquinone “synthesized through simple chemical procedures” from thymoquinone 17Reference 17In vitroIn vitro potential antiviral SARS-CoV-19 activity of natural product thymohydroquinone and dithymoquinone from Nigella sativaView study →. Its practical route into people is not as an isolate at all but as a minor component of black seed oil.
Patents: not yet researched.
Toxicity & Safety
Thymohydroquinone carries a moderate flag, and the reason is candour rather than a documented harm: there is no mammalian toxicology package for this isolate at all — no repeat-dose study, no genotoxicity battery, no reproductive study, no human exposure data. What is documented is a mechanism that argues against assuming safety. The same two-electron chemistry that makes it a good radical scavenger makes it a redox-cycling hydroquinone, and in the one study that looked, thymohydroquinone acted as a prooxidant and damaged isolated plasmid DNA in the presence of free Cu²⁺ or Fe²⁺–EDTA 7Reference 7Antioxidant and prooxidant effects of thymoquinone and its hydroquinone metaboliteView study →. Hydroquinones as a chemical class attract this scrutiny, which is why the closely related arbutin is flagged the same way here.
None of that is an argument against black seed oil, which has a long dietary history and in which thymohydroquinone is a minor constituent 4,
- Dietary exposure is longstanding and small. As a ~3% component of Nigella sativa seed essential oil, ordinary culinary and supplemental black-seed intake delivers only trace amounts.
- No human safety data whatsoever. No trial, no pharmacokinetics, no ADME, no repeat-dose or genotoxicity study of the isolated compound in any species.
- Prooxidant potential. With free transition metals present, thymohydroquinone caused oxidative damage to isolated DNA in vitro — the flip side of its antioxidant chemistry.
- Do not read across from thymoquinone. The safety and efficacy record popularly attached to “black seed’s active compound” belongs to a different molecule and does not transfer.
Full Safety & Interactions Detail
Prooxidant / genotoxic potential. Using ESR and isolated plasmid DNA, thymohydroquinone was shown to have two biologically relevant activities — antioxidant and prooxidant — inducing oxidative DNA damage in the presence of free Cu²⁺ or Fe²⁺–EDTA. Notably, the Fe²⁺ effect disappeared without EDTA, which means the finding is chelation-dependent and may not reflect physiological iron handling 7Reference 7Antioxidant and prooxidant effects of thymoquinone and its hydroquinone metaboliteView study →. No cellular or in-vivo genotoxicity work has followed it up.
Cytotoxicity. Thymohydroquinone is cytotoxic to cultured cells at the concentrations used in tumour assays; the one comparative study reported greater toxicity to tumour lines than to L929 fibroblasts, but non-tumour cells were still killed 12Reference 12In vitroThe antitumor activity of thymoquinone and thymohydroquinone in vitro and in vivoView study →. Repeated intratumoral dosing at 5 mg/kg in mice was tolerated well enough to complete the experiment, and the authors suggested higher doses could be tried — but no systemic-toxicity endpoints were reported 12Reference 12In vitroThe antitumor activity of thymoquinone and thymohydroquinone in vitro and in vivoView study →. A computational study predicted high acute toxicity alongside CNS permeability; that is an in-silico prediction, not a measurement 22Reference 22In silico study of thymohydroquinone interaction with blood-brain barrier disrupting proteinsView study →.
Drug interactions. Not assessed. No CYP-inhibition, CYP-induction, P-glycoprotein or protein-binding study exists for thymohydroquinone. Because it is an NQO1 substrate at the other end of the redox couple 13Reference 13NADPH quinone oxidoreductase 1 mediates breast cancer cell resistance to thymoquinone-induced apoptosisView study →, an interaction with NQO1-dependent drugs or with dicoumarol-type NQO1 inhibitors is mechanistically plausible but entirely untested. The sub-micromolar COX-2 and low-micromolar 5-LOX inhibition seen in cell-free assays 14,
Reproductive note (prose only). No reproductive or developmental-toxicity data exist for isolated thymohydroquinone in any species. Pregnancy and lactation decisions belong to the nigella monograph or to a specific product, where intake is actually decided — not to a molecule-level phytochemistry page.
What is not known. Silence here is not a safety finding. The absence of adverse-effect reports for this compound reflects the absence of studies, not a record of tolerability.
Dosage
There is no dose. Thymohydroquinone has never been administered to humans as an isolated compound, in a trial or otherwise, so no oral, topical or parenteral dose can be stated. Every figure in the literature is a laboratory concentration or an animal research dose:
| Setting | Form | Concentration / dose |
|---|---|---|
| COX-2 inhibition (cell-free) | isolate | IC₅₀ 0.1 µM 14Reference 14In vitroIn vitro inhibitory effects of thymol and quinones of Nigella sativa seeds on cyclooxygenase-1- and -2-catalyzed prostaglandin E2 biosynthesesView study → |
| 5-LOX / LTB₄ inhibition (human neutrophils) | isolate | IC₅₀ 4.1 µM 15Reference 15In vitroInhibition of in vitro leukotriene B4 biosynthesis in human neutrophil granulocytes and docking studies of natural quinonesView study → |
| DPPH radical scavenging | isolate | IC₅₀ 2.4 µg/mL 9Reference 9Determination of oxygen radical absorbance capacity of black cumin (Nigella sativa) seed quinone compoundsView study → |
| Antiyeast activity | isolate | MIC 8–128 µg/mL 16Reference 16In vitroIn vitro antifungal effect of black cumin seed quinones against dairy spoilage yeasts at different acidity levelsView study → |
| Cell cytotoxicity assays | isolate | 0.01–0.1 mg/mL 12Reference 12In vitroThe antitumor activity of thymoquinone and thymohydroquinone in vitro and in vivoView study → |
| Murine tumour models | isolate, intratumoral | 5 mg/kg × 4 injections 12Reference 12In vitroThe antitumor activity of thymoquinone and thymohydroquinone in vitro and in vivoView study → |
Human exposure is dietary and indirect. Black seed oil delivers thymohydroquinone at roughly 3% of its essential-oil fraction 4Reference 4In vitroComposition, in vitro antioxidant and antimicrobial activities of essential oil and oleoresins obtained from black cumin seeds (Nigella sativa L.)View study → — and the essential oil is itself only a small share of the seed — so realistic intake from a standard black-seed supplement is in the milligram-or-less range and is not standardised to this compound. If you are dosing anything, you are dosing nigella seed oil, whose own dosing is discussed on the herb page.
These are research concentrations and animal doses, and are not a personal recommendation.
References
- Ghosheh OA, Houdi AA, Crooks PA (1999). High performance liquid chromatographic analysis of the pharmacologically active quinones and related compounds in the oil of the black seed (Nigella sativa L.). Journal of Pharmaceutical and Biomedical Analysis. https://pubmed.ncbi.nlm.nih.gov/10698539/
- El-Fatatry HM (1975). Isolation and structure assignment of an antimicrobial principle from the volatile oil of Nigella sativa L. seeds. Pharmazie. https://pubmed.ncbi.nlm.nih.gov/238225/
- Botnick I, et al. (2012). Distribution of primary and specialized metabolites in Nigella sativa seeds, a spice with vast traditional and historical uses. Molecules. https://pubmed.ncbi.nlm.nih.gov/22922285/
- Singh S, et al. (2014). Composition, in vitro antioxidant and antimicrobial activities of essential oil and oleoresins obtained from black cumin seeds (Nigella sativa L.). BioMed Research International. https://pubmed.ncbi.nlm.nih.gov/24689064/
- Tiruppur Venkatachallam SK, et al. (2010). Chemical composition of Nigella sativa L. seed extracts obtained by supercritical carbon dioxide. Journal of Food Science and Technology. https://pubmed.ncbi.nlm.nih.gov/23572692/
- Krause ST, et al. (2021). The biosynthesis of thymol, carvacrol, and thymohydroquinone in Lamiaceae proceeds via cytochrome P450s and a short-chain dehydrogenase. Proceedings of the National Academy of Sciences. https://pubmed.ncbi.nlm.nih.gov/34930840/
- Mizuno M, Fukuhara K (2022). Antioxidant and prooxidant effects of thymoquinone and its hydroquinone metabolite. Biological & Pharmaceutical Bulletin. https://pubmed.ncbi.nlm.nih.gov/36047210/
- Sakib R, et al. (2023). Antioxidant properties of thymoquinone, thymohydroquinone and black cumin (Nigella sativa L.) seed oil: scavenging of superoxide radical studied using cyclic voltammetry, DFT and single crystal X-ray diffraction. Antioxidants. https://pubmed.ncbi.nlm.nih.gov/36978853/
- Tesarova H, et al. (2011). Determination of oxygen radical absorbance capacity of black cumin (Nigella sativa) seed quinone compounds. Natural Product Communications. https://pubmed.ncbi.nlm.nih.gov/21425677/
- Jukic M, et al. (2007). In vitro acetylcholinesterase inhibitory properties of thymol, carvacrol and their derivatives thymoquinone and thymohydroquinone. Phytotherapy Research. https://pubmed.ncbi.nlm.nih.gov/17186491/
- Burčul F, et al. (2020). Terpenes, phenylpropanoids, sulfur and other essential oil constituents as inhibitors of cholinesterases. Current Medicinal Chemistry. https://pubmed.ncbi.nlm.nih.gov/29600750/
- Ivankovic S, et al. (2006). The antitumor activity of thymoquinone and thymohydroquinone in vitro and in vivo. Experimental Oncology. https://pubmed.ncbi.nlm.nih.gov/17080016/
- Sutton KM, Doucette CD, Hoskin DW (2012). NADPH quinone oxidoreductase 1 mediates breast cancer cell resistance to thymoquinone-induced apoptosis. Biochemical and Biophysical Research Communications. https://pubmed.ncbi.nlm.nih.gov/22960073/
- Marsik P, et al. (2005). In vitro inhibitory effects of thymol and quinones of Nigella sativa seeds on cyclooxygenase-1- and -2-catalyzed prostaglandin E2 biosyntheses. Planta Medica. https://pubmed.ncbi.nlm.nih.gov/16142638/
- Landa P, et al. (2013). Inhibition of in vitro leukotriene B4 biosynthesis in human neutrophil granulocytes and docking studies of natural quinones. Natural Product Communications. https://pubmed.ncbi.nlm.nih.gov/23472470/
- Halamova K, et al. (2010). In vitro antifungal effect of black cumin seed quinones against dairy spoilage yeasts at different acidity levels. Journal of Food Protection. https://pubmed.ncbi.nlm.nih.gov/21219751/
- Esharkawy ER, Almalki F, Hadda TB (2022). In vitro potential antiviral SARS-CoV-19 activity of natural product thymohydroquinone and dithymoquinone from Nigella sativa. Bioorganic Chemistry. https://pubmed.ncbi.nlm.nih.gov/35026560/
- Judan Cruz KG, et al. (2024). Natural compound-induced downregulation of antimicrobial resistance and biofilm-linked genes in wastewater Aeromonas species. Frontiers in Cellular and Infection Microbiology. https://pubmed.ncbi.nlm.nih.gov/39469451/
- Takada M, et al. (1979). On the metabolic detoxication of thymol in rabbit and man. Journal of Toxicological Sciences. https://pubmed.ncbi.nlm.nih.gov/548583/
- Hahn V, et al. (2013). Two different primary oxidation mechanisms during biotransformation of thymol by gram-positive bacteria of the genera Nocardia and Mycobacterium. Applied Microbiology and Biotechnology. https://pubmed.ncbi.nlm.nih.gov/22828982/
- Karimi A, Meiners T, Böttcher C (2022). Metabolite profiling and bioassay-guided fractionation of Zataria multiflora Boiss. hydroethanolic leaf extracts for identification of broad-spectrum pre- and postharvest antifungal agents. Molecules. https://pubmed.ncbi.nlm.nih.gov/36558036/
- Shah FH, et al. (2020). In silico study of thymohydroquinone interaction with blood-brain barrier disrupting proteins. Future Science OA. https://pubmed.ncbi.nlm.nih.gov/33312701/
- Moussa C, et al. (1997). Microbial models of mammalian metabolism. Fungal metabolism of phenolic and nonphenolic p-cymene-related drugs and prodrugs. I. Metabolites of thymoxamine. Drug Metabolism and Disposition. https://pubmed.ncbi.nlm.nih.gov/9172947/
- Haddad JG, et al. (2019). Ayapana triplinervis essential oil and its main component thymohydroquinone dimethyl ether inhibit Zika virus at doses devoid of toxicity in zebrafish. Molecules. https://pubmed.ncbi.nlm.nih.gov/31547527/
- Ali BH, Blunden G (2003). Pharmacological and toxicological properties of Nigella sativa. Phytotherapy Research. https://pubmed.ncbi.nlm.nih.gov/12722128/
- Svishchuk OA, Visotskii MM (1970). [Synthesis of thymohydroquinone]. Farmatsevtychnyi Zhurnal. https://pubmed.ncbi.nlm.nih.gov/5505177/
- Flaig W, de Jong (1960). [Comparison of the effect of thymoquinone and thymohydroquinone with that of 2,4-dinitrophenol on the metabolism of yeasts (Saccharomyces cerevisiae)]. Archiv für Mikrobiologie. https://pubmed.ncbi.nlm.nih.gov/13700109/



