
Compound Monograph
Senecionine
Senecionine is the archetypal toxic pyrrolizidine alkaloid — a macrocyclic diester of ragwort, coltsfoot and butterbur. CYP3A4 converts it in the liver into a reactive pyrrole that destroys the sinusoidal endothelial cells lining the blood vessels, which is how pyrrolizidine poisoning becomes veno-occlusive liver disease. It sits at the dangerous end of a class whose potencies span a thousandfold.

Sources · 8
Where Does It Come From?
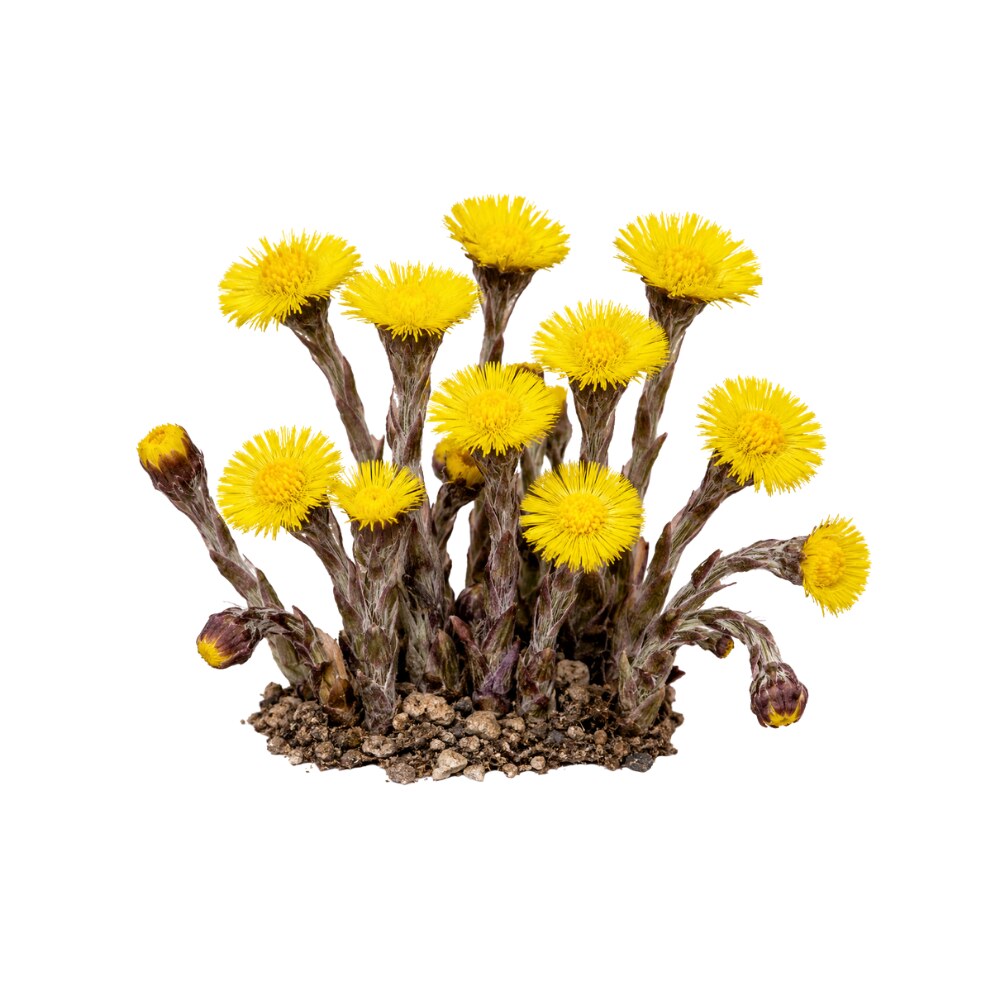
Senecionine is a naturally occurring retronecine-type dehydropyrrolizidine alkaloid (macrocyclic diester), found in Coltsfoot, Butterbur and 6 other sources. It is flagged as toxic and a known carcinogen.
Concentration
Content by Source
Concentrations not reported. No percent-dry-weight or mg/g figures have been published for this compound in its source plants.
Senecionine at a Glance
Senecionine is the pyrrolizidine alkaloid the rest of the class is measured against. It is a macrocyclic diester of retronecine, named for Senecio — the ragworts and groundsels that poison livestock — and it occurs alongside its N-oxide in coltsfoot, butterbur and comfrey’s wider relatives.
Structurally it belongs to the most dangerous subtype of an unevenly dangerous class. Assayed side by side in the same genotoxicity test, sixteen pyrrolizidine alkaloids spanned roughly a thousandfold in potency, with macrocyclic diesters like senecionine at the top and the 7-hydroxy monoesters such as lycopsamine at the bottom 11Reference 11AnimalStructure/activity relationships of the genotoxic potencies of sixteen pyrrolizidine alkaloids assayed for the induction of somatic mutation and recombination in wing cells of Drosophila melanogaster — animal modelView study →. Grouping them all as “PAs” is regulatory convenience, not chemistry.
Its toxicology is unusually well resolved for a plant toxin. Human liver CYP3A4 converts senecionine into a reactive dehydropyrrolizidine that attacks proteins and DNA, and the same enzyme also makes the N-oxide 1Reference 1In vitroRole of cytochrome P450IIIA4 in the metabolism of the pyrrolizidine alkaloid senecionine in human liver — in vitroView study →. What that reactive metabolite kills first is not the hepatocyte that made it but the sinusoidal endothelial cell next door — which is precisely why pyrrolizidine poisoning presents as hepatic veno-occlusive disease, a blockage of the liver’s small blood vessels, rather than as ordinary hepatitis 2Reference 2AnimalThe pyrrolizidine alkaloid senecionine induces CYP-dependent destruction of sinusoidal endothelial cells and cholestasis in mice — mouse in vivoView study →.
The mechanism is shared with the other 1,2-unsaturated pyrrolizidines, and it is set out here in full rather than repeated across senkirkine, lycopsamine and intermedine.
What Makes It the Dangerous Kind
Two structural features have to be present for a pyrrolizidine alkaloid to be a poison, and senecionine has both in their most potent arrangement.
The first is a 1,2-unsaturated necine base — a double bond in the bicyclic core. Without it there is no metabolic activation and no toxicity, which is why coltsfoot’s other alkaloid, tussilagine, is harmless while senecionine is not, despite both being pyrrolizidines.
The second is how the base is esterified. Macrocyclic diesters, in which two ester links close a ring across the molecule, are the most genotoxic; open diesters come next; monoesters are least. The comparison was done directly, dosing sixteen alkaloids orally in the Drosophila wing-spot assay: all but one were genotoxic, but potency ranged across about three orders of magnitude, macrocyclic diesters at the top, 7-hydroxy monoesters at the bottom, and the ranking agreed with rodent hepatotoxicity 11Reference 11AnimalStructure/activity relationships of the genotoxic potencies of sixteen pyrrolizidine alkaloids assayed for the induction of somatic mutation and recombination in wing cells of Drosophila melanogaster — animal modelView study →. Senecionine is a macrocyclic diester.
The N-oxide is not an escape. Plants store much of their senecionine as senecionine N-oxide, which is not itself reactive but is reduced back to the free alkaloid in the gut, so analyses that measure only free bases understate the real exposure 7,
Bioactivation: CYP3A4 Makes the Poison
Senecionine is not toxic as it arrives. It is made toxic by the liver.
Human liver microsomes convert it into two major products: dehydropyrrolizidine (DHP), the reactive pyrrole that does the damage, and senecionine N-oxide, which is a detoxification product. Both reactions are catalysed by the same enzyme. Mechanism-based inactivators of CYP3A4 (gestodene, triacetyloleandomycin) markedly inhibited both, an antibody against CYP3A4 abolished DHP formation entirely in a low-activity liver sample and cut it by 90% in a high-activity one, and the rate of DHP production correlated almost perfectly with nifedipine oxidation, the classical CYP3A4 marker reaction 1Reference 1In vitroRole of cytochrome P450IIIA4 in the metabolism of the pyrrolizidine alkaloid senecionine in human liver — in vitroView study →.
The variation between people is the striking part. Across the human liver samples tested there was a 30-fold difference in DHP formation and a 25-fold difference in N-oxidation between the poorest and the best metaboliser 1Reference 1In vitroRole of cytochrome P450IIIA4 in the metabolism of the pyrrolizidine alkaloid senecionine in human liver — in vitroView study →. Since CYP3A4 activity is itself modulated by dozens of drugs and foods, that variability is a plausible reason why identical pyrrolizidine exposures produce such different outcomes — though nobody has demonstrated this clinically.
Once formed, DHP is an electrophile with two binding partners: proteins, giving the pyrrole-protein adducts now used as a human exposure biomarker 14,
The Cell That Dies First
The most illuminating recent work explains why pyrrolizidine liver injury looks the way it does. Senecionine was given to mice at an acutely toxic dose and the liver watched by intravital two-photon microscopy. What appeared was necrosis of the liver sinusoidal endothelial cells in the pericentral zone, with sinusoidal marker proteins in the serum and platelet aggregation in the damaged regions 2Reference 2AnimalThe pyrrolizidine alkaloid senecionine induces CYP-dependent destruction of sinusoidal endothelial cells and cholestasis in mice — mouse in vivoView study →.
The elegant part is the control experiment. Senecionine applied directly to freshly isolated sinusoidal endothelial cells was not cytotoxic even at 500 µM — but after pre-incubation with primary hepatocytes, which activate it, the resulting medium killed those same endothelial cells with an EC₅₀ around 22 µM. Mice lacking cytochrome-P450 reductase showed no liver injury at all 2Reference 2AnimalThe pyrrolizidine alkaloid senecionine induces CYP-dependent destruction of sinusoidal endothelial cells and cholestasis in mice — mouse in vivoView study →. So the poison is manufactured in the hepatocyte and exported to the endothelium next door.
That is hepatic sinusoidal obstruction syndrome — historically veno-occlusive disease — in mechanistic form: destroy the lining of the small hepatic veins and the blood cannot leave the liver. The same study found delayed uptake and elimination of a fluorescent bile-salt analogue and disturbed expression of bile-salt transporters, adding cholestasis to the picture 2Reference 2AnimalThe pyrrolizidine alkaloid senecionine induces CYP-dependent destruction of sinusoidal endothelial cells and cholestasis in mice — mouse in vivoView study →.
Inside the hepatocyte, senecionine kills by a mitochondrial route: loss of membrane potential, cytochrome-c release, mitochondrial JNK activation and caspase-3-mediated apoptosis, preceded by dramatic fragmentation of the mitochondria. Blocking that fission pharmacologically, or deleting the fission protein Drp1 from hepatocytes, protected mice from senecionine liver injury 3Reference 3AnimalInhibition of Drp1 protects against senecionine-induced mitochondria-mediated apoptosis in primary hepatocytes and in mice — mouse in vivoView study →.
A Pyrrolizidine in a Plant That Never Made It
One unusual route deserves stating, because it is a real hazard for anyone gathering wild plants. Elephant’s head lousewort (Pedicularis groenlandica) is a root hemiparasite, and it takes senecionine up directly from a Senecio host plant and carries it in its own tissue. The uptake was demonstrated for this species by name 18Reference 18Uptake of host plant alkaloids by root parasitic Pedicularis speciesView study →.
The plant does not have the biosynthetic machinery to make pyrrolizidine alkaloids — it is simply plumbed into something that does. A specimen growing on Senecio triangularis carries senecionine; one growing elsewhere does not; and the two are indistinguishable by eye. Alkaloid content in a wildcrafted plant can therefore be a property of its neighbours rather than of its species.
What It's Used For
Senecionine has no therapeutic pharmacology and no dose. Its literature is mechanism, exposure assessment and analytical chemistry.
The best-mapped pyrrolizidine hepatotoxicity in the literature. Bioactivation is CYP3A4-dependent in human liver, producing DHP and the N-oxide with 25–30-fold variation between individuals 1Reference 1In vitroRole of cytochrome P450IIIA4 in the metabolism of the pyrrolizidine alkaloid senecionine in human liver — in vitroView study →.
In mice, an acutely toxic dose produced pericentral sinusoidal endothelial cell necrosis, raised sinusoidal marker proteins and platelet aggregation; the killing required hepatocyte activation (no direct toxicity to endothelial cells at 500 µM, EC₅₀ ~22 µM after activation) and did not occur at all in P450-reductase-deficient mice, alongside delayed bile-salt handling and transporter deregulation 2Reference 2AnimalThe pyrrolizidine alkaloid senecionine induces CYP-dependent destruction of sinusoidal endothelial cells and cholestasis in mice — mouse in vivoView study →.
In primary mouse and human hepatocytes, senecionine caused mitochondrial membrane-potential collapse, cytochrome-c release, JNK translocation and caspase-3 apoptosis with striking mitochondrial fragmentation; Drp1 inhibition and hepatocyte-specific Drp1 knockout both protected mice 3Reference 3AnimalInhibition of Drp1 protects against senecionine-induced mitochondria-mediated apoptosis in primary hepatocytes and in mice — mouse in vivoView study →.
Comparative work in human HepaRG cells places retronecine-type alkaloids including senecionine among the more potent apoptosis inducers, acting after a single 24-hour exposure where otonecine-type senkirkine needed 14 days of repeated dosing 4Reference 4In vitroStructure-dependent induction of apoptosis by hepatotoxic pyrrolizidine alkaloids in the human hepatoma cell line HepaRG: Single versus repeated exposure — in vitroView study →.
Gap: all in-vivo work is rodent. The human record is a class record — hepatic sinusoidal obstruction syndrome from pyrrolizidine-containing herbs and contaminated grain — not senecionine dosed to people, which will never be studied.
Senecionine has no dedicated carcinogenicity bioassay; the class does. Riddelliine, a closely related macrocyclic diester, was carcinogenic in the standard two-year rodent programme at 1 mg/kg by gavage: liver haemangiosarcomas in 86% of male and 76% of female rats, enough early deaths that the male study was terminated at week 72, plus hepatocellular adenomas and eight distinct DNA adducts in liver tissue after three to six months 10Reference 10AnimalToxicology and carcinogenesis studies of riddelliine (CAS NoView study →.
Coltsfoot’s own carcinogenicity study, in which 8 of 12 rats on a high-coltsfoot diet developed hepatic haemangioendothelial sarcoma, attributed the effect to senkirkine rather than to senecionine 5Reference 5AnimalCarcinogenic activity of coltsfoot, Tussilago farfara L. — rat in vivoView study →.
For senecionine itself the evidence is structural and mechanistic: it is a 1,2-unsaturated macrocyclic diester, the most genotoxic subtype in a sixteen-alkaloid comparison spanning about a thousandfold 11Reference 11AnimalStructure/activity relationships of the genotoxic potencies of sixteen pyrrolizidine alkaloids assayed for the induction of somatic mutation and recombination in wing cells of Drosophila melanogaster — animal modelView study →, and its activation product forms DHP-DNA adducts, the common mechanism behind pyrrolizidine carcinogenicity 17Reference 17ReviewMetabolism, genotoxicity, and carcinogenicity of comfrey — reviewView study →. Regulators assess 1,2-unsaturated PAs as one group on exactly this reasoning 12Reference 12ReviewRisk assessment of pyrrolizidine alkaloids in food of plant and animal origin — reviewView study →.
Gap: no compound-specific bioassay, so the carcinogenicity claim is read across from riddelliine and from mechanism. Given the shared activation chemistry, that read-across is well founded, but it is a read-across.
The practical subject. Senecionine and senkirkine are the pyrrolizidines detected analytically in coltsfoot 6Reference 6Sensitive determination of pyrrolizidine alkaloids in Tussilago farfara L. by field-amplified, sample-stacking, sweeping micellar electrokinetic chromatography — analyticalView study → and, with their N-oxides, in butterbur rhizome 7Reference 7Simultaneous investigation of sesquiterpenes, pyrrolizidine alkaloids and N-oxides in Butterbur (Petasites hybridus) with an offline 2D-combination of HPLC-UV and LC-MMI-ToF-MS — analyticalView study →.
Regulatory pressure has pushed detection limits to a few parts per billion, and a purpose-built method for the commercial butterbur extract Ze 339 quantified five alkaloids down to 2 ppb and found none present in the tested batches 8Reference 8UPLC TOF MS for sensitive quantification of naturally occurring pyrrolizidine alkaloids in Petasites hybridus extract (Ze 339) — analyticalView study → — the distinction between a raw PA-bearing plant and an industrially depleted extract, which matters for butterbur specifically.
Exposure is not confined to herbs. Pyrrolizidine alkaloids reach food through honey, milk and contaminated crops, with herbal teas identified as the main dietary source in the European assessment 12Reference 12ReviewRisk assessment of pyrrolizidine alkaloids in food of plant and animal origin — reviewView study →, and a 2020 study found senkirkine, senecionine and senecionine N-oxide in stream water beside invasive butterbur stands at about 70 ng/L, rising tenfold after heavy rain, and up to 230 ng/L in seepage water from groundwater wells 9Reference 9The invasive butterbur contaminates stream and seepage water in groundwater wells with toxic pyrrolizidine alkaloids — analyticalView study →.
In exposed people, pyrrole-protein and pyrrole-haemoglobin adducts now serve as blood biomarkers of pyrrolizidine exposure and injury 14,
Gap: no measured senecionine content is available for the coltsfoot or butterbur material actually sold; the analytical papers report method performance and detection, not survey concentrations.
None. No therapeutic application of senecionine has been proposed, and the alkaloid is studied purely as a toxin and analytical marker.
Mechanisms
| Target / pathway | Effect | Relevant to |
|---|---|---|
| CYP3A4 | Oxidation to the reactive pyrrole DHP (bioactivation) and to the N-oxide (detoxification); 25–30-fold interindividual range | Everything downstream; interaction potential |
| Gut microbial reduction | Senecionine N-oxide reduced back to the free alkaloid | Why N-oxides are not a safe form |
| Cellular proteins | Pyrrole-protein adducts — also the human exposure biomarker | Toxicity and biomonitoring |
| DNA | DHP-DNA adducts, the common pyrrolizidine carcinogenic mechanism | Genotoxicitycarcinogenicity |
| Liver sinusoidal endothelial cells | Killed by hepatocyte-generated metabolite (EC₅₀ ~22 µM), not by senecionine itself | Veno-occlusive disease / sinusoidal obstruction syndrome |
| Mitochondrial fission (Drp1) | Fragmentation, cytochrome-c release, JNK and caspase-3 apoptosis | Hepatocyte death; Drp1 loss is protective |
| Bile-salt transporters (Abcb11, Abcc1) | Delayed uptake and elimination, transcriptional deregulation | Cholestasis |
One fact organises the table: the liver builds the poison, and the neighbouring blood vessel absorbs it.
Pharmacokinetics
Senecionine’s disposition is dominated by first-pass metabolism, and the balance between its two CYP3A4 routes decides the outcome: DHP formation is bioactivation, N-oxidation is detoxification, and both rates vary 25–30-fold between human livers 1Reference 1In vitroRole of cytochrome P450IIIA4 in the metabolism of the pyrrolizidine alkaloid senecionine in human liver — in vitroView study →. The N-oxide is not a terminal metabolite in practice, because gut microbiota reduce it back to the parent alkaloid, which is why an N-oxide-rich plant is not a safer plant 9,
Clinical Trials
None, and none is possible. The human evidence consists of poisoning case series across the pyrrolizidine class, biomarker studies in exposed patients 14,
| Completed | Planned | Terminated | Preclinical |
|---|---|---|---|
| None | — | — | Extensive mechanistic toxicology; class carcinogenicity bioassay (riddelliine) |
Last checked: September 2026.
Isolate vs. Plant Studies
Unusually for a plant constituent, the isolate work is the relevant work: purified senecionine in human liver microsomes 1Reference 1In vitroRole of cytochrome P450IIIA4 in the metabolism of the pyrrolizidine alkaloid senecionine in human liver — in vitroView study →, in primary hepatocytes and mice 2,
Where plant context does matter is in mixtures and N-oxides. Plants deliver senecionine alongside seneciphylline, senkirkine and the N-oxides of each 7,
Its Role in Plants
Pyrrolizidine alkaloids are chemical defence against herbivores, and their biosynthesis is one of the better-understood specialised pathways in plants: it begins with homospermidine synthase, an enzyme recruited from the housekeeping enzyme deoxyhypusine synthase, which is why the pathway has arisen independently in several unrelated families 16Reference 16ReviewPyrrolizidine alkaloids: biosynthesis, biological activities and occurrence in crop plants — reviewView study →. In Senecio the alkaloids are made in the roots and transported as N-oxides to the shoots, where they are stored.
Some insects have turned the defence around: arctiid moths and other specialists sequester senecionine from their food plants, store it, and use it for their own protection and as a precursor to pheromones. The alkaloid that poisons a cow is a resource to a moth.
Prevalence in Nature
Senecionine is a hallmark alkaloid of the tribe Senecioneae in the Asteraceae. Its namesake genus Senecio — ragworts and groundsels — is the classic source and the cause of most livestock pyrrolizidine poisoning worldwide.
Among herbs, it is detected analytically in coltsfoot (Tussilago farfara) together with senkirkine 6Reference 6Sensitive determination of pyrrolizidine alkaloids in Tussilago farfara L. by field-amplified, sample-stacking, sweeping micellar electrokinetic chromatography — analyticalView study →, and in butterbur (Petasites hybridus) rhizome with its N-oxide alongside senkirkine and seneciphylline 7,
Two routes carry it outside the plants that make it. The first is the food chain: pyrrolizidine alkaloids appear in honey from PA-bearing forage, in milk, and as crop contaminants, with herbal teas the main dietary source in European assessment 12Reference 12ReviewRisk assessment of pyrrolizidine alkaloids in food of plant and animal origin — reviewView study →. The second is root hemiparasitism — elephant’s head lousewort takes senecionine directly from a Senecio host 18Reference 18Uptake of host plant alkaloids by root parasitic Pedicularis speciesView study →.
Discovery & Synthesis
Senecionine was characterised from Senecio early in the twentieth century, part of the chemical investigation of the livestock poisonings that made ragwort a notifiable weed in several countries, and it takes its name from the genus. It became the reference compound of pyrrolizidine toxicology: the 1991 demonstration that human CYP3A4 performs both its activation and its detoxification was done on senecionine 1Reference 1In vitroRole of cytochrome P450IIIA4 in the metabolism of the pyrrolizidine alkaloid senecionine in human liver — in vitroView study →, and it is one of the standard alkaloids in structure-activity comparisons 4,
It is not manufactured. Senecionine is isolated from plant material for use as an analytical standard and a research toxin, and the commercial interest runs entirely the other way — toward reference standards accurate enough to detect it at parts per billion in food, herbal extracts and water 8,
Toxicity & Safety
Senecionine is flagged toxic and carcinogen, and both are literal. It is a hepatotoxin with a mapped mechanism and a member of a class assessed as genotoxic carcinogens with no threshold.
The Injury It Causes
Pyrrolizidine liver injury is hepatic sinusoidal obstruction syndrome — the small hepatic veins are blocked by damage to their endothelial lining, and blood cannot drain from the liver. It presents with abdominal pain, ascites, hepatomegaly and jaundice, and it can be fatal or leave permanent damage. The mechanism is set out above: hepatocytes make the reactive metabolite and the neighbouring endothelial cells die of it 2Reference 2AnimalThe pyrrolizidine alkaloid senecionine induces CYP-dependent destruction of sinusoidal endothelial cells and cholestasis in mice — mouse in vivoView study →. Cholestasis accompanies it 2Reference 2AnimalThe pyrrolizidine alkaloid senecionine induces CYP-dependent destruction of sinusoidal endothelial cells and cholestasis in mice — mouse in vivoView study →. There is no antidote.
Exposure Limits
There is no safe intake. The European chronic assessment for 1,2-unsaturated pyrrolizidine alkaloids works from a BMDL₁₀ of 237 µg/kg body weight per day derived from riddelliine data, and names herbal teas and teas as the main dietary source 12Reference 12ReviewRisk assessment of pyrrolizidine alkaloids in food of plant and animal origin — reviewView study →; a proposed acute reference dose of 1 µg/kg body weight per day was later derived from a sub-acute rat study and supported by human poisoning cases 13Reference 13ReviewRisk assessment of short-term intake of pyrrolizidine alkaloids in food: derivation of an acute reference dose — reviewView study →. Regulatory limits for herbal medicines now sit at levels requiring parts-per-billion analytical methods 8Reference 8UPLC TOF MS for sensitive quantification of naturally occurring pyrrolizidine alkaloids in Petasites hybridus extract (Ze 339) — analyticalView study →.
Who Is At Risk
Anyone consuming a pyrrolizidine-bearing plant internally, in any preparation — hot water does not exclude these alkaloids, and neither does alcohol. Because bioactivation runs through CYP3A4, and that enzyme’s activity varies 30-fold between people and is modulated by many drugs, exposure and susceptibility are both variable 1Reference 1In vitroRole of cytochrome P450IIIA4 in the metabolism of the pyrrolizidine alkaloid senecionine in human liver — in vitroView study →; this is mechanistically obvious and clinically unstudied. Children, pregnant women (the alkaloids cross the placenta as a class) and people with existing liver disease are the conventional high-risk groups. Plants containing senecionine should not be taken internally, and the decision about any particular herb belongs on that herb’s page, where preparation and alkaloid content are known.
- Hepatotoxic with no safe intake. CYP3A4 converts it to a reactive pyrrole that destroys the lining of the liver’s small veins, causing sinusoidal obstruction syndrome.
- Genotoxic carcinogen by class. Its close relative riddelliine caused liver haemangiosarcomas in most treated rats at 1 mg/kg.
- The N-oxide is not a safe form. Gut bacteria reduce it back to the alkaloid, so analyses that ignore N-oxides understate exposure.
- Susceptibility varies 30-fold. Bioactivation depends on CYP3A4 activity, which differs widely between people and is altered by many drugs.
- Exposure reaches beyond herbs. Honey, milk, contaminated crops, and stream and well water near butterbur stands.
- Depleted extracts are a different product. The commercial butterbur extract Ze 339 had no detectable pyrrolizidine alkaloids down to 2 ppb.
Dosage
There is no dose, and no preparation should be taken to obtain senecionine. The relevant numbers are limits and measured contamination.
| Context | Figure |
|---|---|
| Proposed acute reference dose (PA class) | 1 µg/kg body weight/day 13Reference 13ReviewRisk assessment of short-term intake of pyrrolizidine alkaloids in food: derivation of an acute reference dose — reviewView study → |
| Chronic assessment point of departure (BMDL₁₀, riddelliine) | 237 µg/kg body weight/day 12Reference 12ReviewRisk assessment of pyrrolizidine alkaloids in food of plant and animal origin — reviewView study → |
| Butterbur extract Ze 339, five PAs | None detected, limit of quantification 2 ppb 8Reference 8UPLC TOF MS for sensitive quantification of naturally occurring pyrrolizidine alkaloids in Petasites hybridus extract (Ze 339) — analyticalView study → |
| Stream water beside butterbur | ~70 ng/L, tenfold higher after rain 9Reference 9The invasive butterbur contaminates stream and seepage water in groundwater wells with toxic pyrrolizidine alkaloids — analyticalView study → |
| Seepage water, groundwater wells | Up to 230 ng/L 9Reference 9The invasive butterbur contaminates stream and seepage water in groundwater wells with toxic pyrrolizidine alkaloids — analyticalView study → |
| Riddelliine rodent carcinogenic dose (class read-across) | 1 mg/kg by gavage → haemangiosarcoma in 76–86% of rats 10Reference 10AnimalToxicology and carcinogenesis studies of riddelliine (CAS NoView study → |
References
- Miranda CL, Reed RL, Guengerich FP, et al. (1991). Role of cytochrome P450IIIA4 in the metabolism of the pyrrolizidine alkaloid senecionine in human liver — in vitro. Carcinogenesis. https://pubmed.ncbi.nlm.nih.gov/2009596/
- Hessel-Pras S, Braeuning A, Guenther G, et al. (2020). The pyrrolizidine alkaloid senecionine induces CYP-dependent destruction of sinusoidal endothelial cells and cholestasis in mice — mouse in vivo. Arch Toxicol. https://pubmed.ncbi.nlm.nih.gov/31606820/
- Yang X, Wang H, Ni HM, et al. (2017). Inhibition of Drp1 protects against senecionine-induced mitochondria-mediated apoptosis in primary hepatocytes and in mice — mouse in vivo. Redox Biol. https://pubmed.ncbi.nlm.nih.gov/28282614/
- Waizenegger J, Braeuning A, Templin M, et al. (2018). Structure-dependent induction of apoptosis by hepatotoxic pyrrolizidine alkaloids in the human hepatoma cell line HepaRG: Single versus repeated exposure — in vitro. Food Chem Toxicol. https://pubmed.ncbi.nlm.nih.gov/29458164/
- Hirono I, Mori H, Culvenor CC (1976). Carcinogenic activity of coltsfoot, Tussilago farfara L. — rat in vivo. Gan. https://pubmed.ncbi.nlm.nih.gov/1269853/
- Cao K, Xu Y, Mu X, et al. (2016). Sensitive determination of pyrrolizidine alkaloids in Tussilago farfara L. by field-amplified, sample-stacking, sweeping micellar electrokinetic chromatography — analytical. J Sep Sci. https://pubmed.ncbi.nlm.nih.gov/27673325/
- Aydın AA, Letzel T (2013). Simultaneous investigation of sesquiterpenes, pyrrolizidine alkaloids and N-oxides in Butterbur (Petasites hybridus) with an offline 2D-combination of HPLC-UV and LC-MMI-ToF-MS — analytical. J Pharm Biomed Anal. https://pubmed.ncbi.nlm.nih.gov/23906985/
- Schenk A, Siewert B, Toff S, et al. (2015). UPLC TOF MS for sensitive quantification of naturally occurring pyrrolizidine alkaloids in Petasites hybridus extract (Ze 339) — analytical. J Chromatogr B Analyt Technol Biomed Life Sci. https://pubmed.ncbi.nlm.nih.gov/26094206/
- Kisielius V, Hama JR, Skrbic N, et al. (2020). The invasive butterbur contaminates stream and seepage water in groundwater wells with toxic pyrrolizidine alkaloids — analytical. Sci Rep. https://pubmed.ncbi.nlm.nih.gov/33188248/
- National Toxicology Program (2003). Toxicology and carcinogenesis studies of riddelliine (CAS No. 23246-96-0) in F344/N rats and B6C3F1 mice (gavage studies) — animal in vivo. Natl Toxicol Program Tech Rep Ser. https://pubmed.ncbi.nlm.nih.gov/12844193/
- Frei H, Lüthy J, Brauchli J, et al. (1992). Structure/activity relationships of the genotoxic potencies of sixteen pyrrolizidine alkaloids assayed for the induction of somatic mutation and recombination in wing cells of Drosophila melanogaster — animal model. Chem Biol Interact. https://pubmed.ncbi.nlm.nih.gov/1643665/
- Dusemund B, Nowak N, Sommerfeld C, et al. (2018). Risk assessment of pyrrolizidine alkaloids in food of plant and animal origin — review. Food Chem Toxicol. https://pubmed.ncbi.nlm.nih.gov/29524571/
- Eckert E, Lepper H, Hintzsche H (2023). Risk assessment of short-term intake of pyrrolizidine alkaloids in food: derivation of an acute reference dose — review. Food Addit Contam Part A Chem Anal Control Expo Risk Assess. https://pubmed.ncbi.nlm.nih.gov/36794362/
- Ruan J, Gao H, Li N, et al. (2015). Blood pyrrole-protein adducts — a biomarker of pyrrolizidine alkaloid-induced liver injury in humans — review. J Environ Sci Health C Environ Carcinog Ecotoxicol Rev. https://pubmed.ncbi.nlm.nih.gov/26398275/
- Ma J, Zhang W, He Y, et al. (2021). Clinical application of pyrrole-hemoglobin adducts as a biomarker of pyrrolizidine alkaloid exposure in humans — in patients. Arch Toxicol. https://pubmed.ncbi.nlm.nih.gov/33210216/
- Schramm S, Köhler N, Rozhon W (2019). Pyrrolizidine alkaloids: biosynthesis, biological activities and occurrence in crop plants — review. Molecules. https://pubmed.ncbi.nlm.nih.gov/30704105/
- Mei N, Guo L, Fu PP, et al. (2010). Metabolism, genotoxicity, and carcinogenicity of comfrey — review. J Toxicol Environ Health B Crit Rev. https://pubmed.ncbi.nlm.nih.gov/21170807/
- Schneider MJ, Stermitz FR (1990). Uptake of host plant alkaloids by root parasitic Pedicularis species. Phytochemistry. https://doi.org/10.1016/0031-9422(90)85021-7



