
Compound Monograph
Isorhamnetin
Isorhamnetin is the 3′-O-methyl ether of quercetin — a dietary flavonol that is also a major in-vivo metabolite of quercetin and rutin in humans, so part of what quercetin "does" may actually run through isorhamnetin. It is the signature flavonol of sea-buckthorn fruit and a principal flavonol of Ginkgo leaf. Methylation gives it somewhat better membrane permeability than quercetin, but oral bioavailability is still limited and every application signal — cardiovascular, anti-inflammatory, metabolic, hepatoprotective, anticancer — is preclinical, with no isolated-molecule human trial.

Sources · 10
Where Does It Come From?
Isorhamnetin is a naturally occurring flavonol (o-methylated), found in Sea buckthorn, Ginkgo, Goldenrod and 7 other sources. It is well tolerated orally (low toxicity).
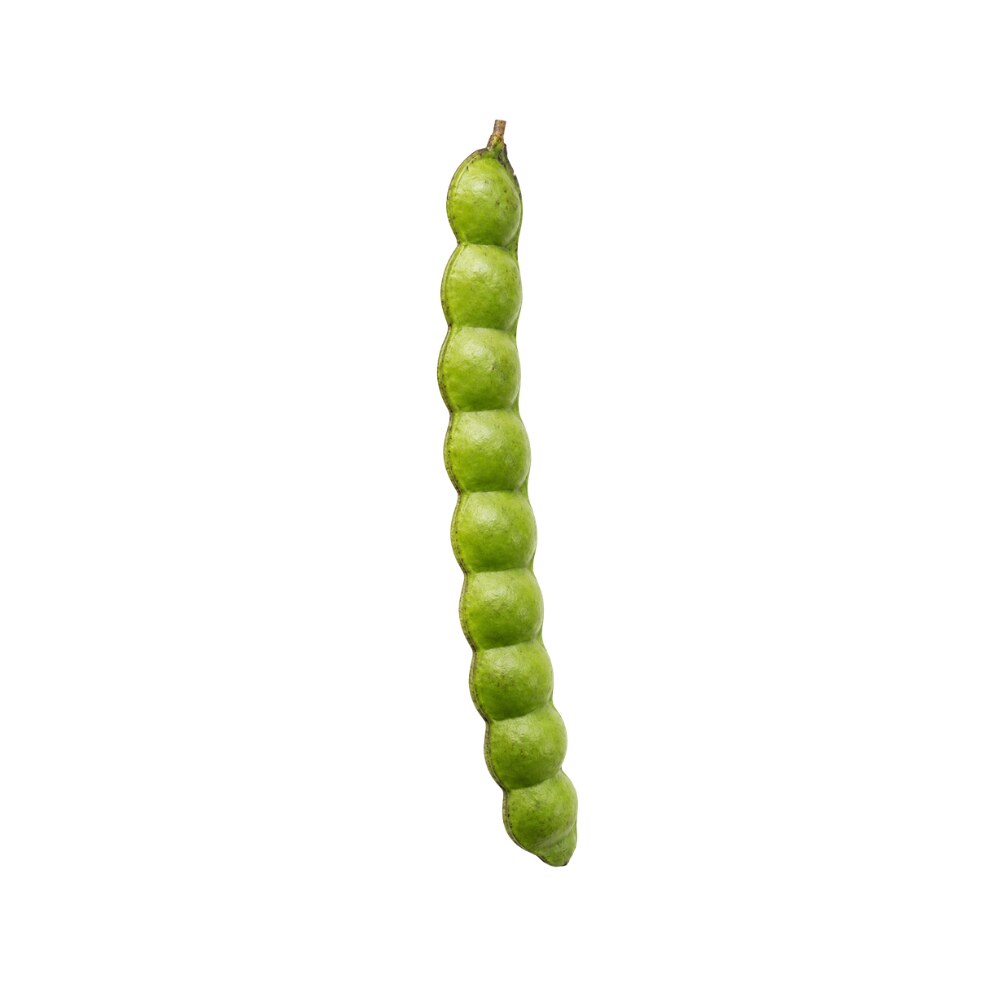 Source African Dream Herb Entada rheedii Herb monograph →
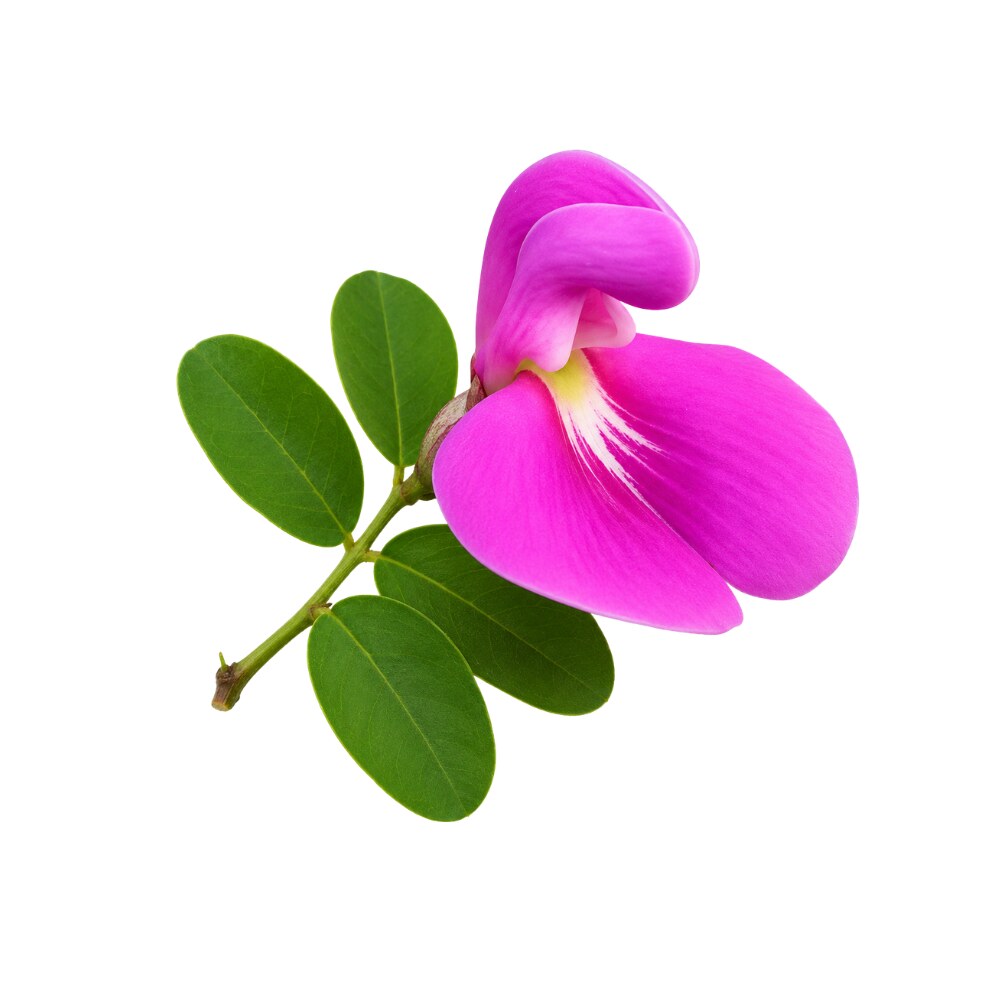 Source Bay Bean Canavalia rosea Herb monograph →
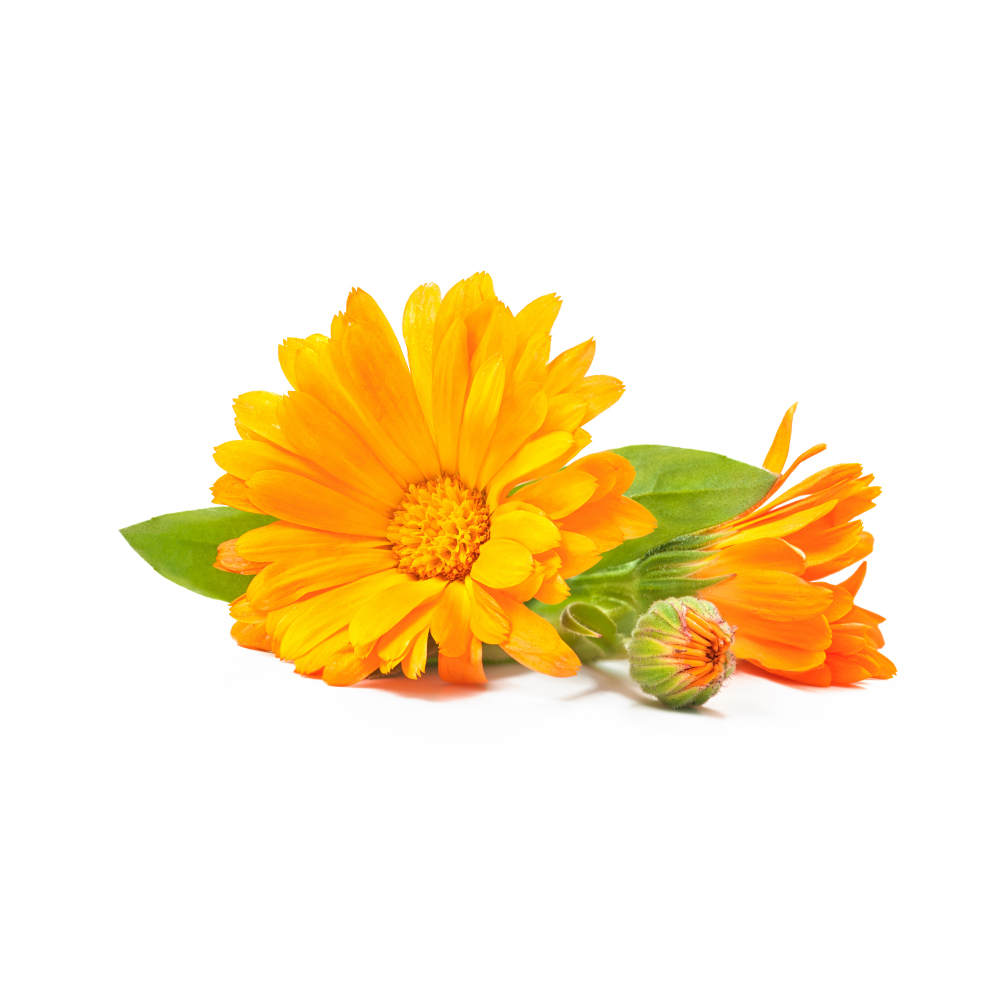 Source Calendula Calendula officinalis Herb monograph →
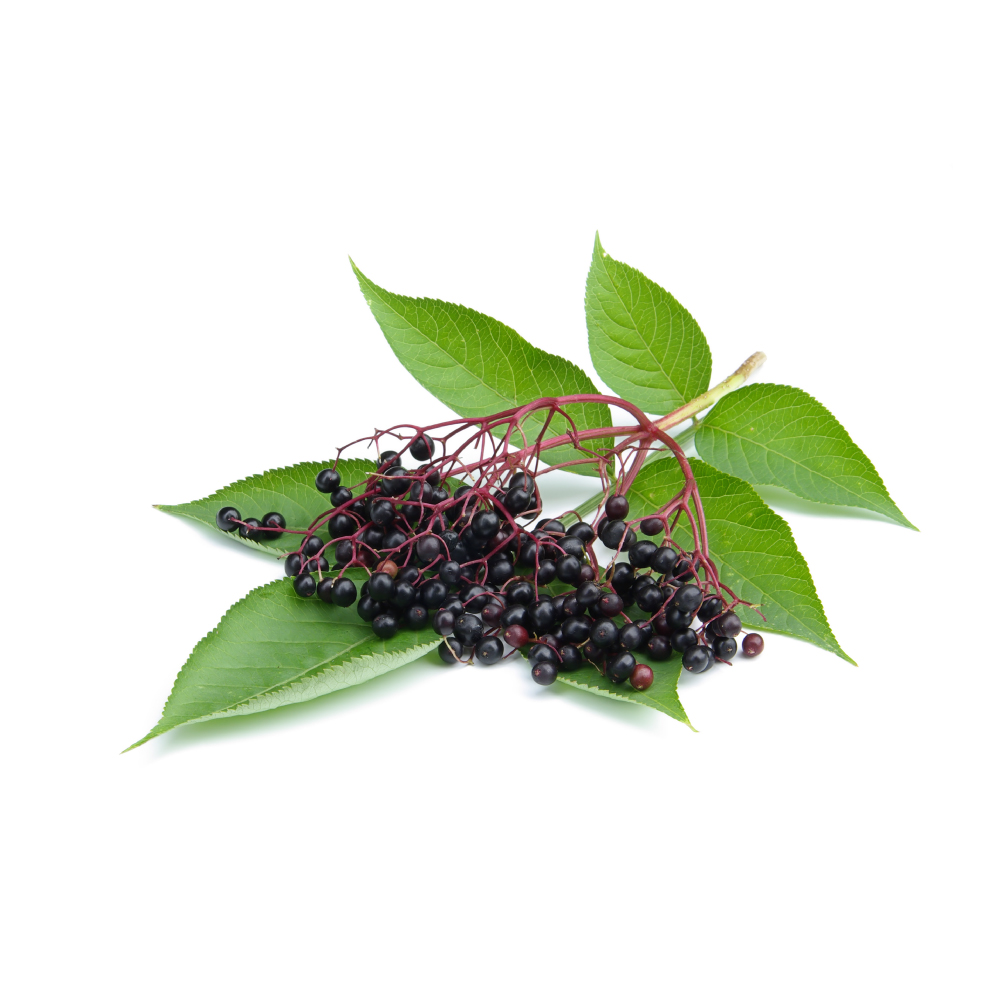 Source Elderberry Sambucus nigra Herb monograph →
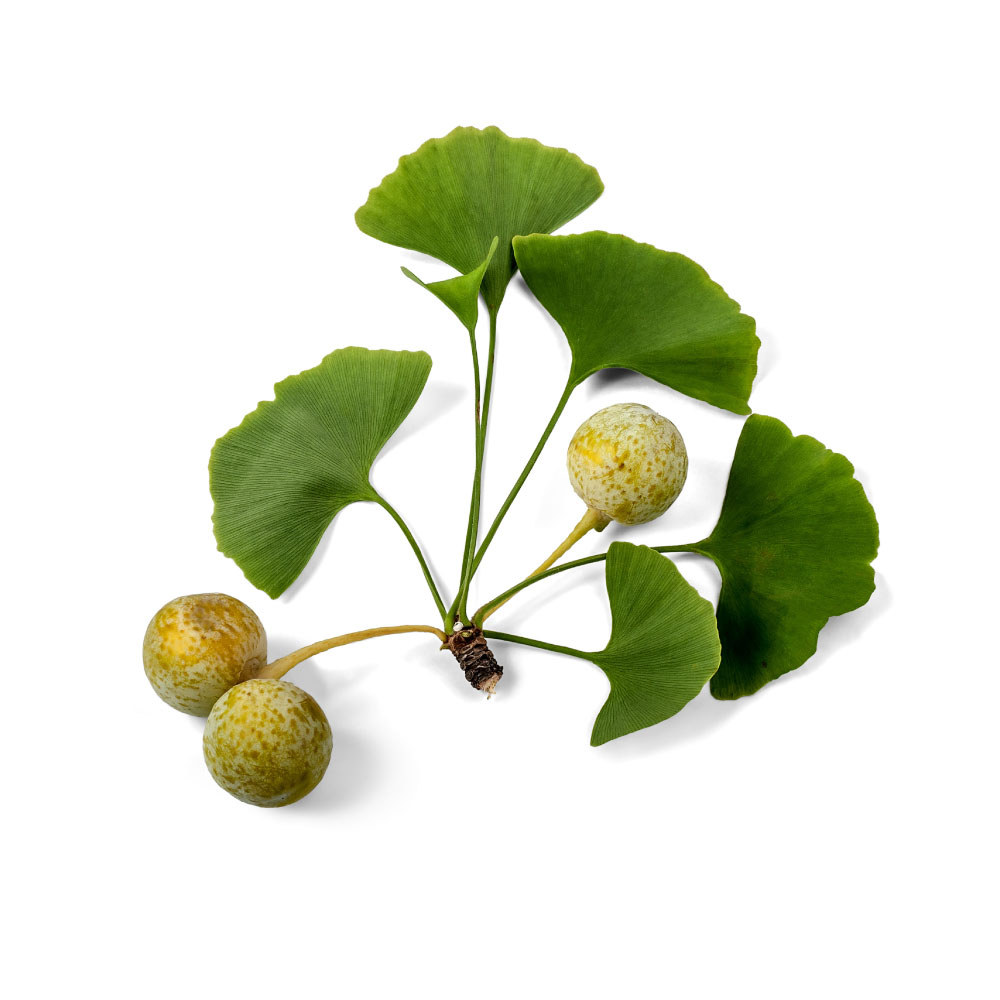 Source Ginkgo Ginkgo biloba Herb monograph →
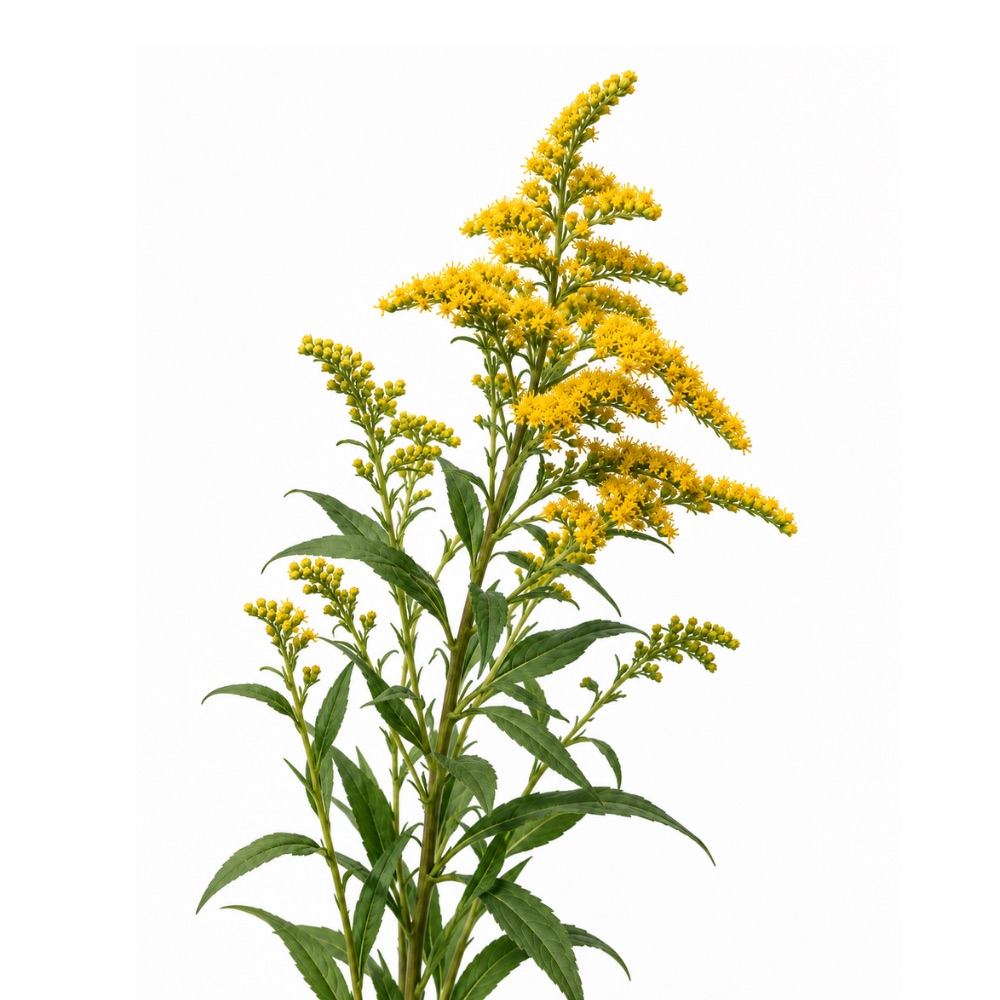 Source Goldenrod Solidago virgaurea Herb monograph →
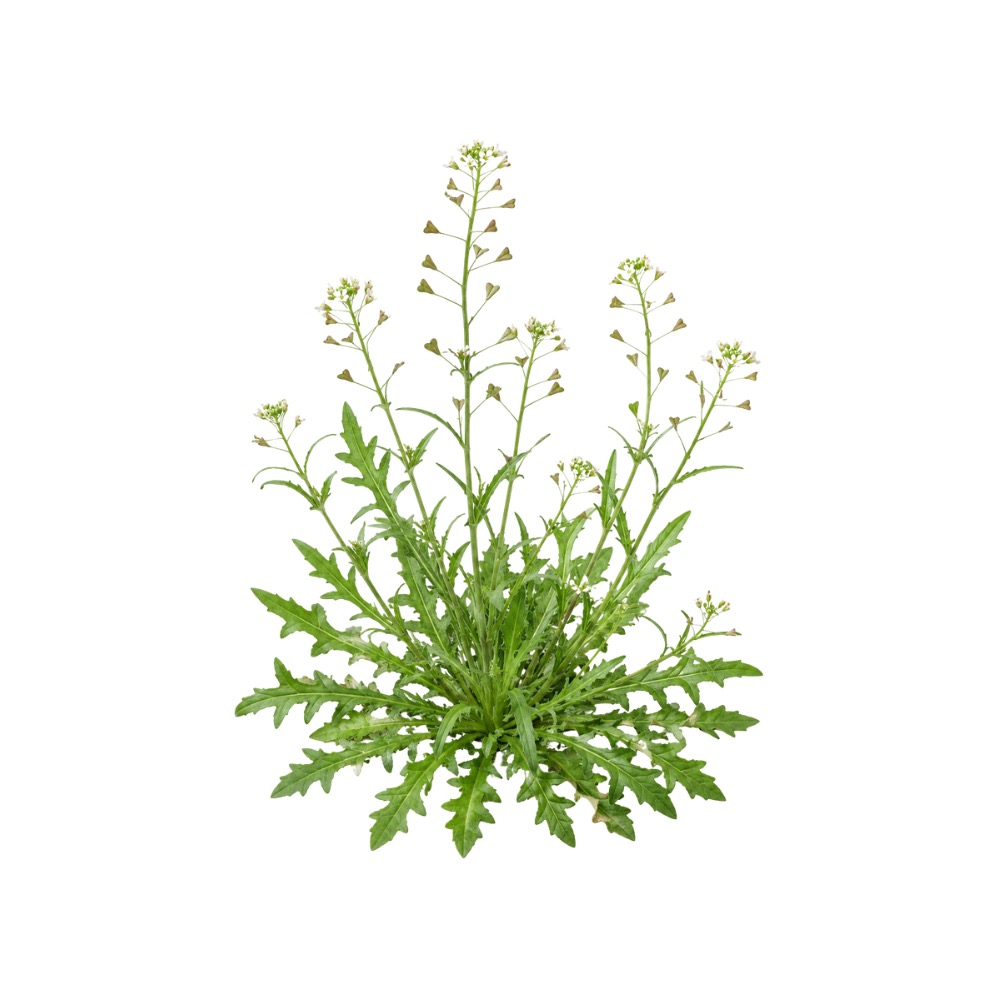 Source Shepherd's Purse Capsella bursa-pastoris Herb monograph →
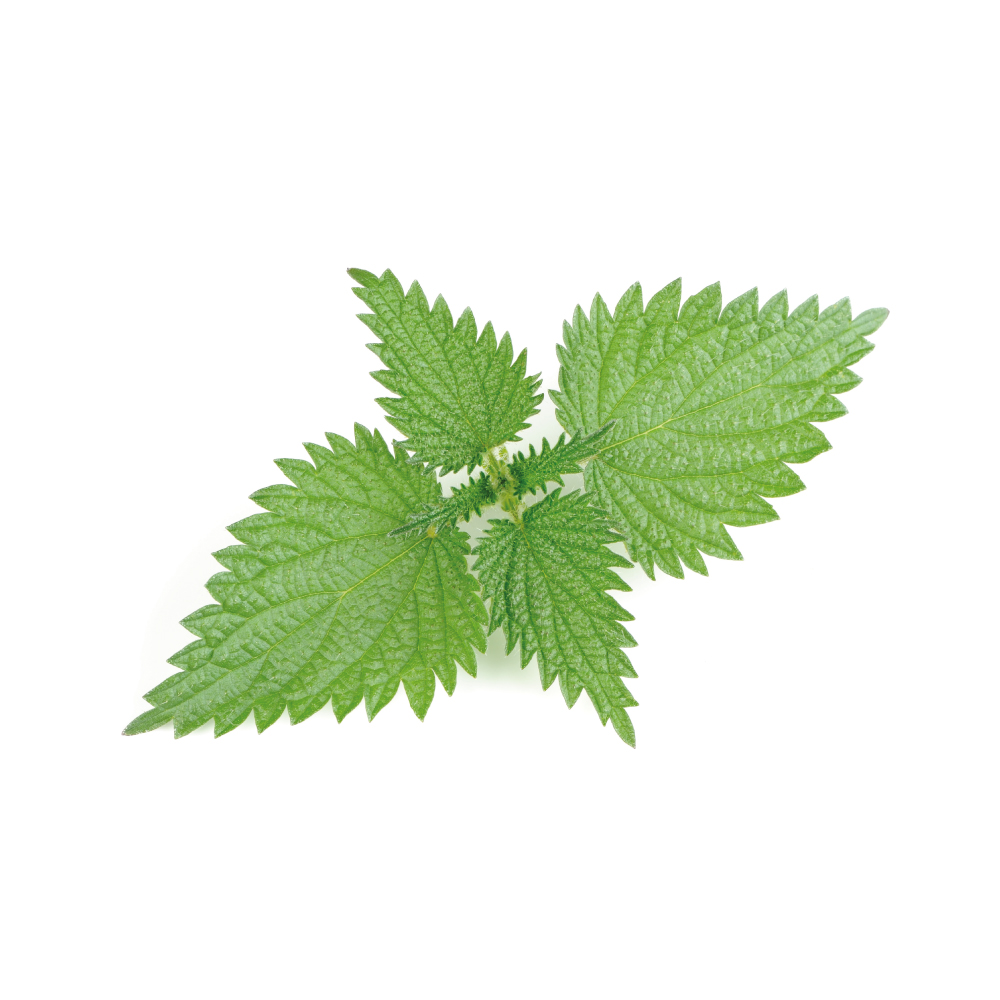 Source Stinging Nettle Urtica dioica Herb monograph →
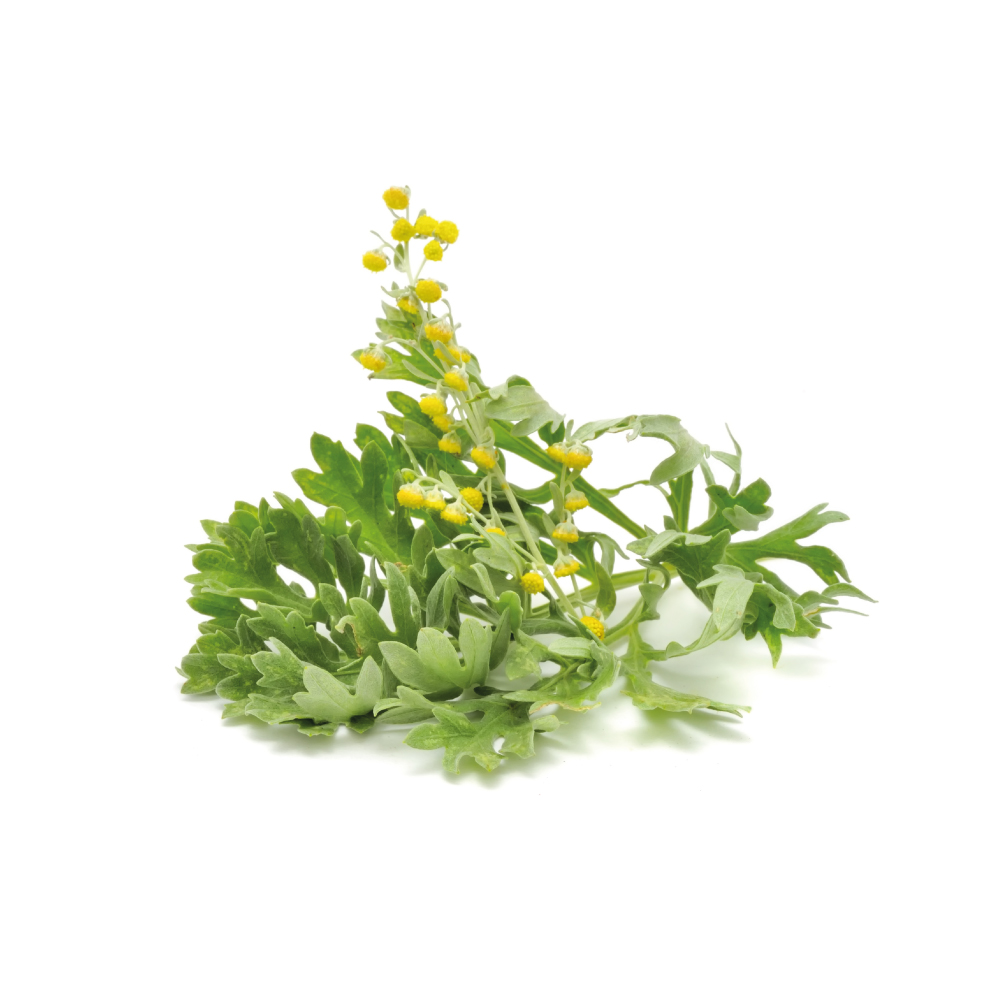 Source Wormwood Artemisia absinthium Herb monograph →
Concentration
Content by Source
Concentrations not reported. No percent-dry-weight or mg/g figures have been published for this compound in its source plants.
Isorhamnetin at a Glance
Isorhamnetin is the 3’-O-methyl ether of quercetin — and also a major human metabolite of quercetin and rutin.
That dual identity is the interesting part: some of what quercetin appears to do in a body may actually be isorhamnetin’s work, since methylation happens rapidly after absorption and the methylated form circulates alongside the parent.
It is also a dietary flavonol in its own right, concentrated in sea buckthorn and mustard greens.
What It's Used For
Isorhamnetin (3′-O-methylquercetin) is a dietary flavonol — quercetin carrying a single methyl group on the 3′ position of its B-ring. That one methyl is why its literature reads two ways at once. In plants isorhamnetin is a widespread flavonol in its own right: the signature flavonol of sea-buckthorn fruit, one of the three principal flavonols of Ginkgo leaf (where it contributes to the radical-scavenging antioxidant fraction of the standardized extract 6Reference 6In vitroPeroxyl radical scavenging activity of Ginkgo biloba extract EGb 761 — in vitroView study →), and a recurring antioxidant constituent across this database — in goldenrod, wormwood, stinging nettle, calendula, elder and African dream herb — almost always stored as glycosides 1Reference 1ReviewIsorhamnetin: A review of pharmacological effects — reviewView study →.
In people it is also a major circulating metabolite of quercetin and rutin: catechol-O-methyltransferase methylates quercetin’s 3′-hydroxyl, so isorhamnetin appears in blood after any quercetin-rich intake and is part of what quercetin’s activity actually reflects 1,
Methylation blocks one of quercetin’s conjugation sites, giving isorhamnetin somewhat better membrane permeability and metabolic stability — but oral bioavailability is still limited, and, as with every flavonol here, the entire applied literature is preclinical: cardiovascular, anti-inflammatory, metabolic, hepatoprotective and anticancer signals from cell and rodent models, with no trial of the isolated molecule in humans 1Reference 1ReviewIsorhamnetin: A review of pharmacological effects — reviewView study →.
Support is an experimental score — weighted by study type (human > animal > in vitro) and volume, tempered for isolate-vs-plant match and bioavailability. A beta, not a validated metric. Scores are held low because there is no isolated-isorhamnetin human trial. Each application links to its write-up.
The broadest and most in-vivo signal. Isolated isorhamnetin given to mice for eight weeks after aortic banding blunted pressure-overload cardiac hypertrophy and fibrosis, an effect traced to blocking PI3K–AKT signaling 9Reference 9AnimalIsorhamnetin protects against cardiac hypertrophy through blocking PI3K–AKT pathway — mouse aortic-banding modelView study →.
In isolated rat hearts it reduced ischemia-reperfusion infarct size and marker-enzyme release (LDH, CK) dose-dependently, limiting cardiomyocyte apoptosis and oxidative stress (↑Bcl-2, ↓Bax/caspase-3, ↓MDA) 10Reference 10AnimalCardioprotective effect of isorhamnetin against myocardial ischemia reperfusion (I/R) injury in isolated rat heart through attenuation of apoptosis — rat modelView study →.
At the vessel wall it protected TNF-α-injured endothelial cells (HUVECs), cutting apoptosis and the adhesion molecules ICAM-1, VCAM-1 and E-selectin via NF-κB suppression while restoring eNOS 8Reference 8In vitroProtective effects of isorhamnetin on apoptosis and inflammation in TNF-α-induced HUVECs injury — in vitroView study →.
The pharmacological review catalogues further anti-atherosclerotic and anti-thrombotic actions 1Reference 1ReviewIsorhamnetin: A review of pharmacological effects — reviewView study →.
Gap: every result is cell or rodent; there is no human cardiovascular trial, and the doses were not bioavailability-matched to what oral intake achieves.
A consistent mechanistic through-line: isolated isorhamnetin dampens NF-κB-driven inflammation. In LPS-challenged mice it lowered TNF-α, IL-1β and IL-6 and reduced tissue injury by downregulating NF-κB signaling 12Reference 12In vitroIsorhamnetin ameliorates LPS-induced inflammatory response through downregulation of NF-κB signaling — in vitro and mouse modelView study →, and in an LPS acute-lung-injury model it attenuated lung edema, MPO activity and cytokine release (also implicating mTOR) 14Reference 14AnimalIsorhamnetin alleviates lipopolysaccharide-induced acute lung injury by inhibiting mTOR signaling pathway — mouse modelView study →. The same NF-κB suppression underlies its endothelial protection 8Reference 8In vitroProtective effects of isorhamnetin on apoptosis and inflammation in TNF-α-induced HUVECs injury — in vitroView study →.
Gap: rodent and cell models only; the anti-inflammatory doses have no human counterpart, and NF-κB inhibition is a shared flavonol mechanism rather than something specific to isorhamnetin.
Isolated isorhamnetin promotes glucose disposal and opposes adiposity in mechanistic models. In cultured myotubes it increased glucose uptake by translocating GLUT4 — notably through the JAK2/STAT pathway, a different route from quercetin’s CaMKKβ/AMPK, and active at low-nanomolar concentrations 7Reference 7In vitroQuercetin and its metabolite isorhamnetin promote glucose uptake through different signalling pathways in myotubes — in vitroView study →. Dedicated reviews summarize anti-diabetic actions (aldose-reductase inhibition, improved insulin signaling, protection against diabetic complications) 2Reference 2In vitroEffects of Isorhamnetin on Diabetes and Its Associated Complications: A Review of In Vitro and In Vivo Studies and a Post Hoc Transcriptome Analysis — reviewView study → and anti-obesity effects (suppressed adipogenesis, PPARγ modulation) 3Reference 3ReviewAnti-Obesity Effects of Isorhamnetin and Isorhamnetin Conjugates — reviewView study →.
Gap: the evidence is cell-based or review-level; there are no clinical glucose or weight outcomes for the isolated molecule.
Isolated isorhamnetin protects the liver across injury models. In a diet-induced NASH mouse it reduced steatosis and fibrosis at 50 mg/kg — cutting hepatic triglyceride and collagen by downregulating lipogenic (SREBP1c/FAS/ACC1) and fibrogenic (TGF-β/collagen-I) programs 11Reference 11AnimalIsorhamnetin Alleviates Steatosis and Fibrosis in Mice with Nonalcoholic Steatohepatitis — mouse modelView study →. In a separate mouse model of chemical liver injury it lowered transaminases and inflammatory cytokines and regulated apoptosis/autophagy via the P38/PPAR-α pathway 5Reference 5AnimalIsorhamnetin: A hepatoprotective flavonoid inhibits apoptosis and autophagy via P38/PPAR-α pathway in mice — mouse modelView study →.
Gap: in-vivo but single-laboratory rodent work with no human data; the NASH finding awaits independent replication.
The broadest but thinnest signal. Isolated isorhamnetin induces apoptosis and cell-cycle arrest across cultured tumor lines: in human bladder-cancer cells it triggered ROS-dependent G2/M arrest and both intrinsic and extrinsic apoptosis through AMPK activation 13Reference 13In vitroIsorhamnetin Induces Cell Cycle Arrest and Apoptosis Via Reactive Oxygen Species-Mediated AMP-Activated Protein Kinase Signaling Pathway Activation in Human Bladder Cancer Cells — in vitroView study →, and a 2024 review catalogues similar in-vitro activity (AMPK/mTOR, PI3K-Akt and EMT effects) in breast, gastric, colon and lung lines 4Reference 4In vitroIsorhamnetin: what is the in vitro evidence for its antitumor potential and beyond? — reviewView study →.
Gap: almost entirely in-vitro at concentrations the poor oral bioavailability makes hard to reach systemically; in-vivo tumor data are sparse and there are no human oncology data 4Reference 4In vitroIsorhamnetin: what is the in vitro evidence for its antitumor potential and beyond? — reviewView study →.
Mechanisms
| Target / pathway | Effect | Relevant to |
|---|---|---|
| PI3K–AKT | Inhibits → ↓cardiac hypertrophy / fibrosis | Cardiovascular |
| NF-κB / MAPK, ICAM-1/VCAM-1 | Suppresses → ↓inflammation, endothelial protection | Anti-inflammatorycardiovascular |
| eNOS | Upregulates → nitric-oxide / endothelial support | Cardiovascular |
| Bcl-2/Bax, caspase-3/9 | Modulates → ↓cardiomyocyte apoptosis (protective) | Cardiovascular |
| GLUT4 via JAK2/STAT | Activates → ↑glucose uptake | Metabolic |
| SREBP1c/FAS/ACC1, PPAR-α | Downregulates lipogenesis / regulates lipid metabolism | Hepatoprotectivemetabolic |
| ROS → AMPK → mTOR/p70S6K | Activates (pro-apoptotic in tumor cells) | Anticancer |
| Radical scavenging (flavonol antioxidant) | Peroxyl/hydroxyl scavenging, ↓lipid peroxidation | General antioxidant |
Pharmacokinetics
Isorhamnetin’s defining pharmacokinetic fact is its relationship to quercetin. It is not only a plant flavonol but a major in-vivo metabolite of quercetin and rutin: catechol-O-methyltransferase (COMT) methylates quercetin’s 3′-hydroxyl, so isorhamnetin circulates after any quercetin-rich intake and is part of what quercetin’s activity actually reflects 1,
Clinical trials
There are essentially no registered trials of isolated isorhamnetin. Its human relevance is indirect — it is one of the circulating metabolites measured in quercetin, sea-buckthorn and Ginkgo trials, which are plant- or parent-molecule exposures and cannot be read as isorhamnetin results. Everything here is preclinical.
| Completed | Planned | Terminated | Preclinical |
|---|---|---|---|
| None(isolated isorhamnetin) | None known | None | Extensive |
Last checked: July 2026.
Toxicity & Safety
Isorhamnetin carries a low toxicity flag. It is a common dietary flavonol — eaten in onions, pears, sea-buckthorn and leafy herbs — and, unusually, it is also generated inside the body from quercetin, so people are chronically and safely exposed to it at dietary levels 1Reference 1ReviewIsorhamnetin: A review of pharmacological effects — reviewView study →. Reviews describe it as well tolerated in animal studies without signature organ toxicity at the doses used, though no formal human safety database exists because the isolated molecule has not been trialled in people 1Reference 1ReviewIsorhamnetin: A review of pharmacological effects — reviewView study →. Like other flavonols it can inhibit drug-metabolizing cytochrome-P450 enzymes and transporters in laboratory systems, so interactions with medications are plausible but not clinically quantified; reasonable caution applies to anyone combining high-dose flavonol supplements with narrow-margin CYP / P-glycoprotein-substrate drugs. Isorhamnetin also shares quercetin’s caveat that most of its striking in-vitro activity — including the pro-apoptotic anticancer effects — occurs at concentrations well above achievable plasma levels, a potency that does not automatically translate into whole-body effect or harm. No isolated-molecule reproductive or developmental toxicity finding was identified in this pass.
Dosage
There is no established human dose for isolated isorhamnetin. Preclinical work spans cell-culture concentrations from low-nanomolar (glucose uptake in myotubes) to tens of micromolar (anticancer apoptosis), and rodent doses in the tens of mg/kg range — for example 50 mg/kg in the NASH model and 100 mg/kg in the cardiac-hypertrophy study 7,
References
- Gong G, Guan YY, Zhang ZL, Rahman K, Wang SJ, Zhou S, Luan X, Zhang H. (2020). Isorhamnetin: A review of pharmacological effects — review. Biomedicine & Pharmacotherapy, 128, 110301. https://pubmed.ncbi.nlm.nih.gov/32502837/
- Kalai FZ, Boulaaba M, Ferdousi F, Isoda H. (2022). Effects of Isorhamnetin on Diabetes and Its Associated Complications: A Review of In Vitro and In Vivo Studies and a Post Hoc Transcriptome Analysis — review. International Journal of Molecular Sciences, 23(2), 704. https://pubmed.ncbi.nlm.nih.gov/35054888/
- González-Arceo M, Gomez-Lopez I, Carr-Ugarte H, et al. (2022). Anti-Obesity Effects of Isorhamnetin and Isorhamnetin Conjugates — review. International Journal of Molecular Sciences, 24(1), 299. https://pubmed.ncbi.nlm.nih.gov/36613743/
- Lei J, Yang Y, Zhou W, et al. (2024). Isorhamnetin: what is the in vitro evidence for its antitumor potential and beyond? — review. Frontiers in Pharmacology, 15, 1309178. https://pubmed.ncbi.nlm.nih.gov/38650631/
- Lu X, Liu T, Chen K, Xia Y, Dai W, Xu S, et al. (2018). Isorhamnetin: A hepatoprotective flavonoid inhibits apoptosis and autophagy via P38/PPAR-α pathway in mice — mouse model. Biomedicine & Pharmacotherapy, 103, 800–811. https://pubmed.ncbi.nlm.nih.gov/29684859/
- Maitra I, Marcocci L, Droy-Lefaix MT, Packer L. (1995). Peroxyl radical scavenging activity of Ginkgo biloba extract EGb 761 — in vitro. Biochemical Pharmacology, 49(11), 1649–1655. https://pubmed.ncbi.nlm.nih.gov/7786306/
- Jiang H, Yamashita Y, Nakamura A, Croft K, Ashida H. (2019). Quercetin and its metabolite isorhamnetin promote glucose uptake through different signalling pathways in myotubes — in vitro. Scientific Reports, 9, 2690. https://pubmed.ncbi.nlm.nih.gov/30804434/
- Chen TL, Zhu GL, He XL, Wang JA. (2015). Protective effects of isorhamnetin on apoptosis and inflammation in TNF-α-induced HUVECs injury — in vitro. International Journal of Clinical and Experimental Pathology, 8(3), 2311–2320. https://pubmed.ncbi.nlm.nih.gov/26045738/
- Gao L, Yao R, Liu Y, Wang Z, Huang Z, Du B, et al. (2017). Isorhamnetin protects against cardiac hypertrophy through blocking PI3K–AKT pathway — mouse aortic-banding model. Molecular and Cellular Biochemistry, 429(1–2), 167–177. https://pubmed.ncbi.nlm.nih.gov/28176246/
- Xu Y, Tang C, Tan S, Duan J, Tian H, Yang Y. (2020). Cardioprotective effect of isorhamnetin against myocardial ischemia reperfusion (I/R) injury in isolated rat heart through attenuation of apoptosis — rat model. Journal of Cellular and Molecular Medicine, 24(11), 6253–6262. https://pubmed.ncbi.nlm.nih.gov/32307912/
- Ganbold M, Owada Y, Ozawa Y, Shimamoto Y, Ferdousi F, Tominaga K, et al. (2019). Isorhamnetin Alleviates Steatosis and Fibrosis in Mice with Nonalcoholic Steatohepatitis — mouse model. Scientific Reports, 9, 16210. https://pubmed.ncbi.nlm.nih.gov/31700054/
- Li Y, Chi G, Shen B, Tian Y, Feng H. (2016). Isorhamnetin ameliorates LPS-induced inflammatory response through downregulation of NF-κB signaling — in vitro and mouse model. Inflammation, 39(4), 1291–1301. https://pubmed.ncbi.nlm.nih.gov/27138362/
- Park C, Cha HJ, Choi EO, Lee H, Hwang-Bo H, Ji SY, et al. (2019). Isorhamnetin Induces Cell Cycle Arrest and Apoptosis Via Reactive Oxygen Species-Mediated AMP-Activated Protein Kinase Signaling Pathway Activation in Human Bladder Cancer Cells — in vitro. Cancers, 11(10), 1494. https://pubmed.ncbi.nlm.nih.gov/31590241/
- Yang B, Ma L, Wei Y, Cui Y, et al. (2022). Isorhamnetin alleviates lipopolysaccharide-induced acute lung injury by inhibiting mTOR signaling pathway — mouse model. Immunopharmacology and Immunotoxicology, 44(3), 387–396. https://pubmed.ncbi.nlm.nih.gov/35306954/



