
Compound Monograph
Scopoletin
Scopoletin (6-methoxy-7-hydroxycoumarin) is a widely distributed plant hydroxycoumarin. Its preclinical research centers on anti-inflammatory (NF-κB/Nrf2), antioxidant, and xanthine-oxidase-mediated urate-lowering activity — with no human trials of the isolate. It is not the hepatotoxic "coumarin" of fragrance nor a warfarin-type anticoagulant.

Sources · 18
Where Does It Come From?
Scopoletin is a naturally occurring coumarin, found in Stinging Nettle, Marshmallow, Passionflower and 15 other sources. It is well tolerated orally (low toxicity).
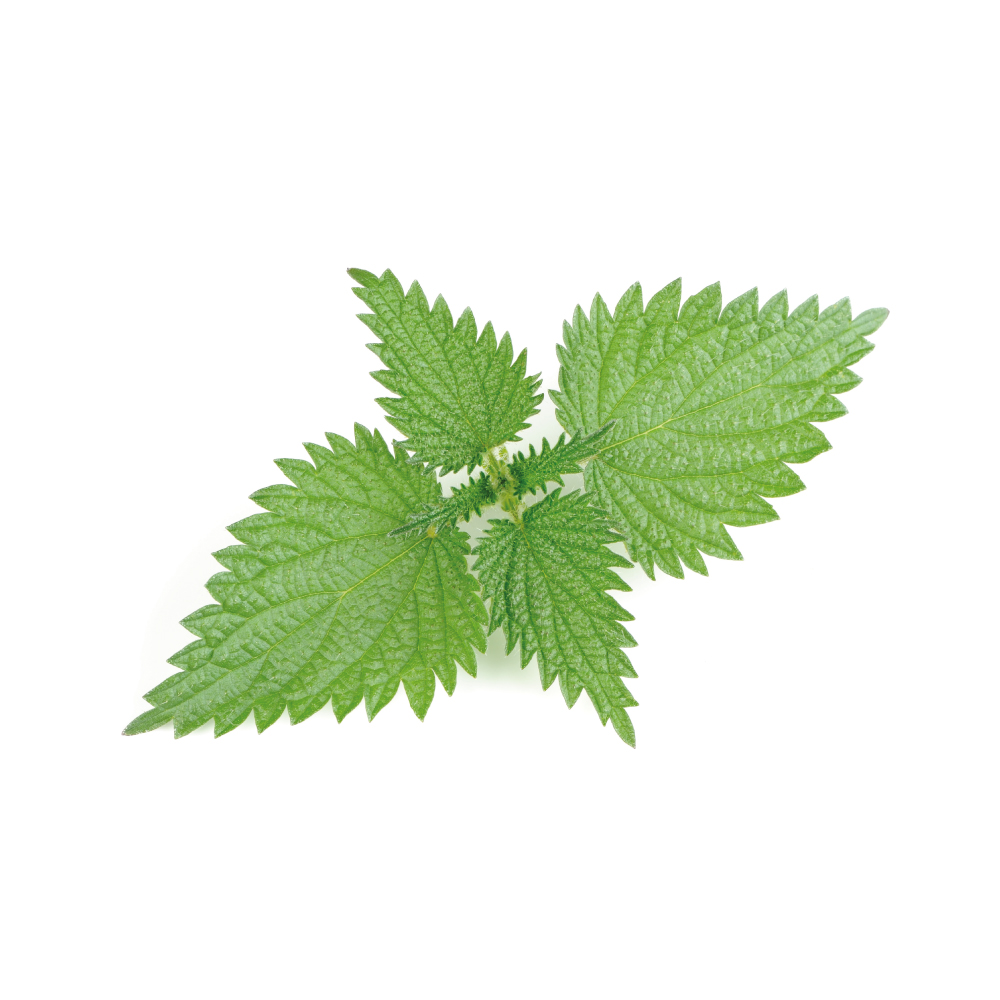 Principal source Stinging Nettle Urtica dioica Herb monograph →
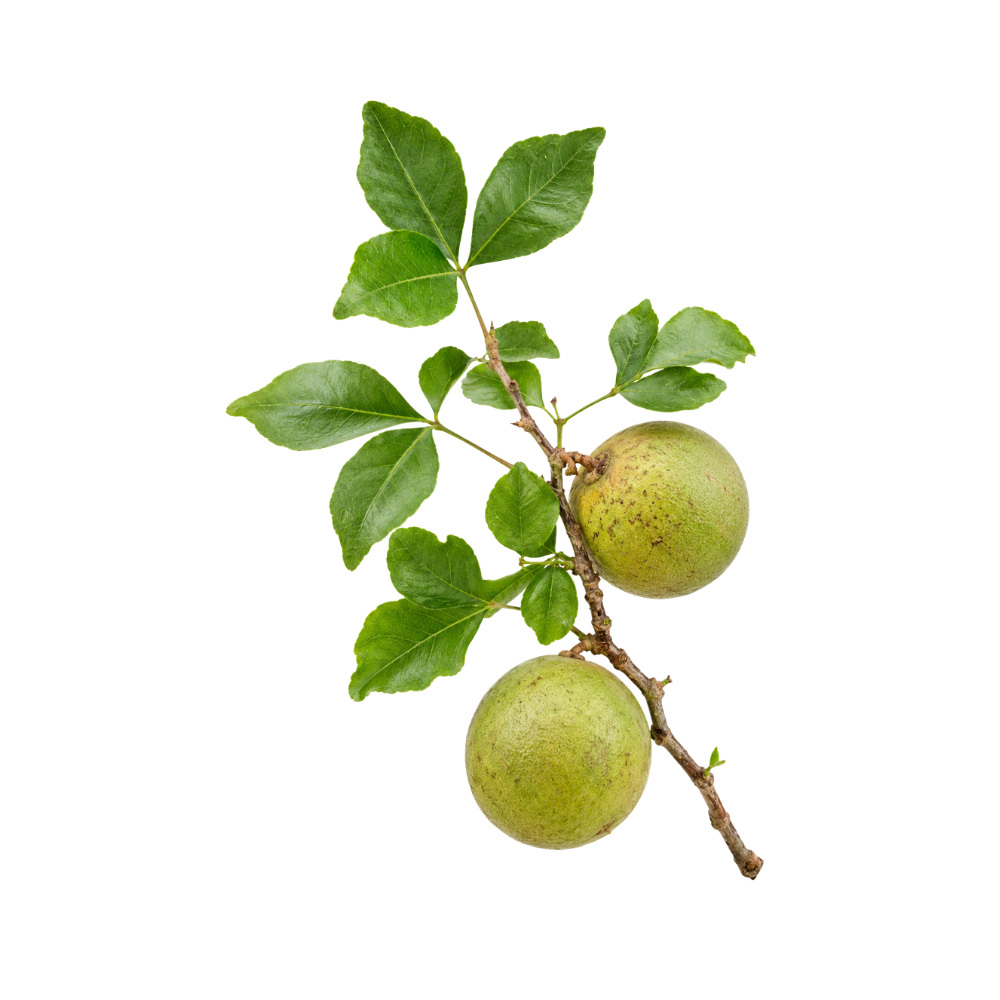 Source Bael Aegle marmelos Herb monograph →
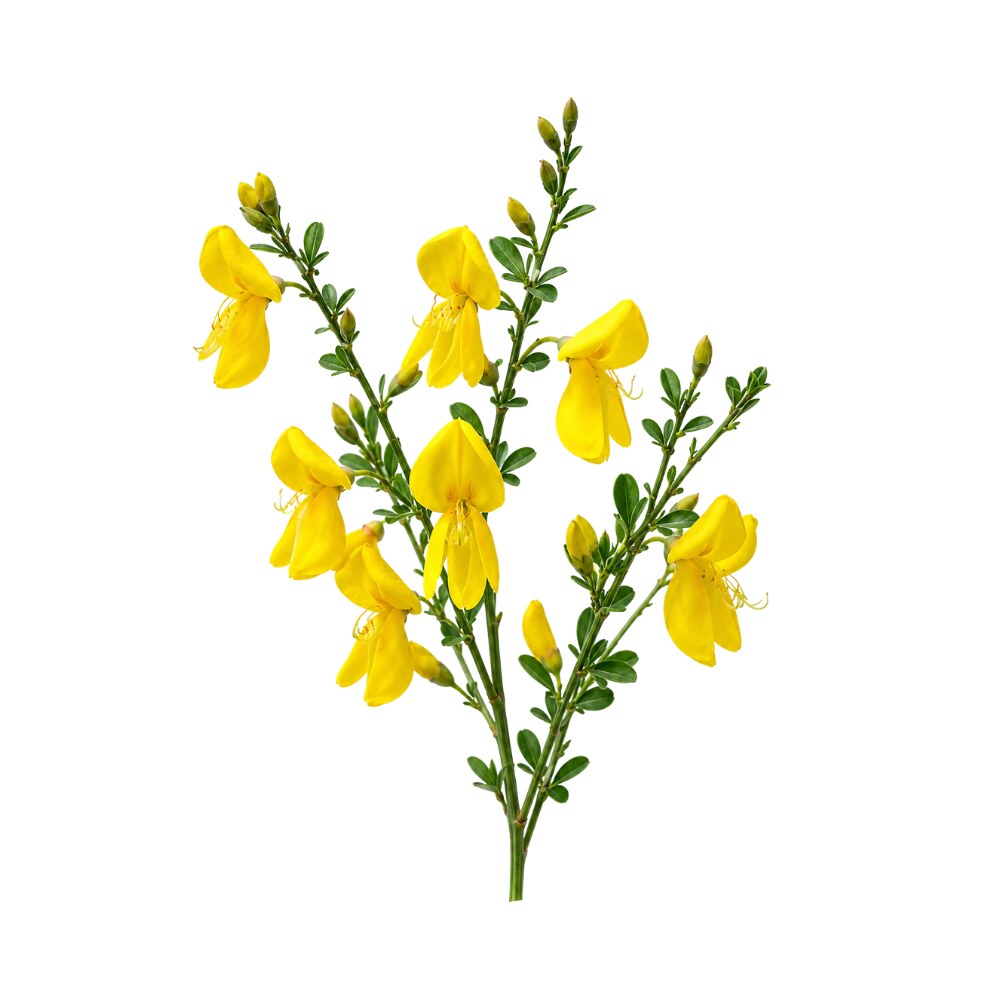 Source Broom Cytisus scoparius Herb monograph →
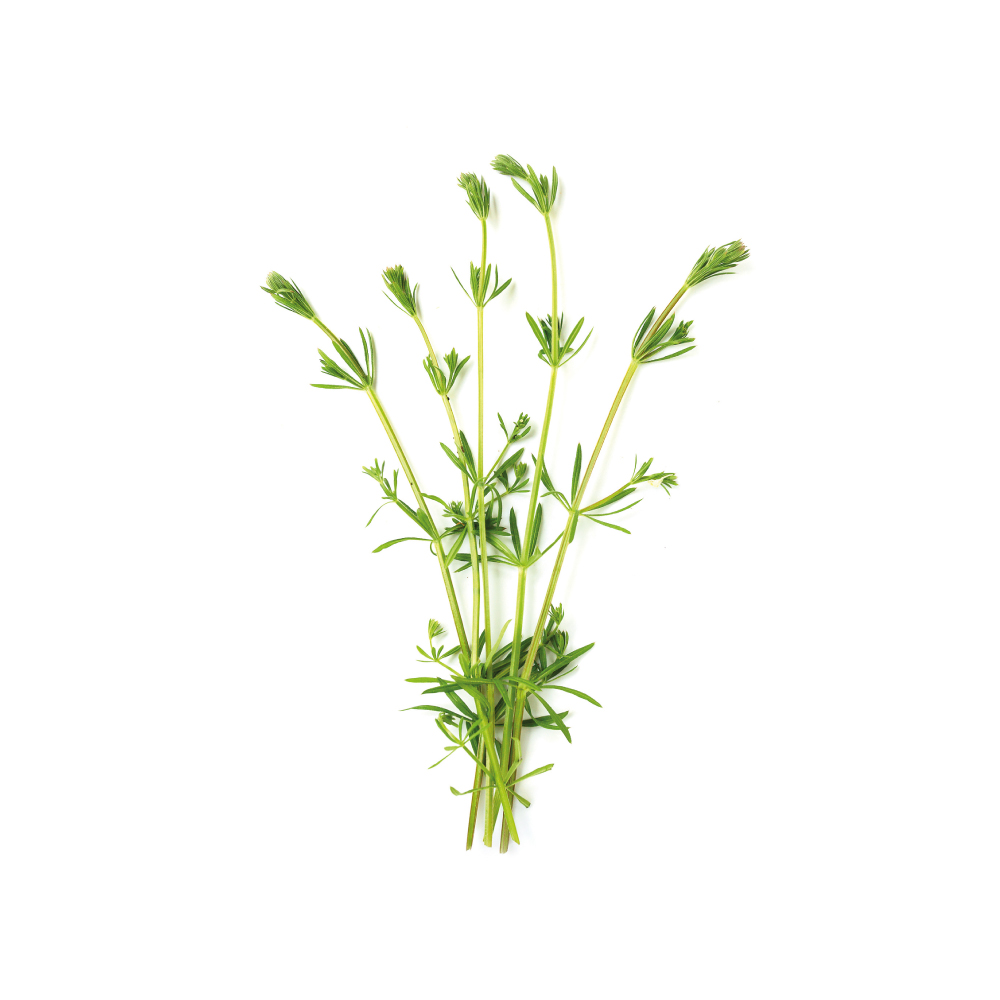 Source Cleavers Galium aparine Herb monograph →
 Source Cramp Bark Viburnum opulus Herb monograph →
 Source Dandelion Taraxacum officinale Herb monograph →
 Source Linden Flower Tilia spp. Herb monograph →
 Source Lobelia Lobelia inflata Herb monograph →
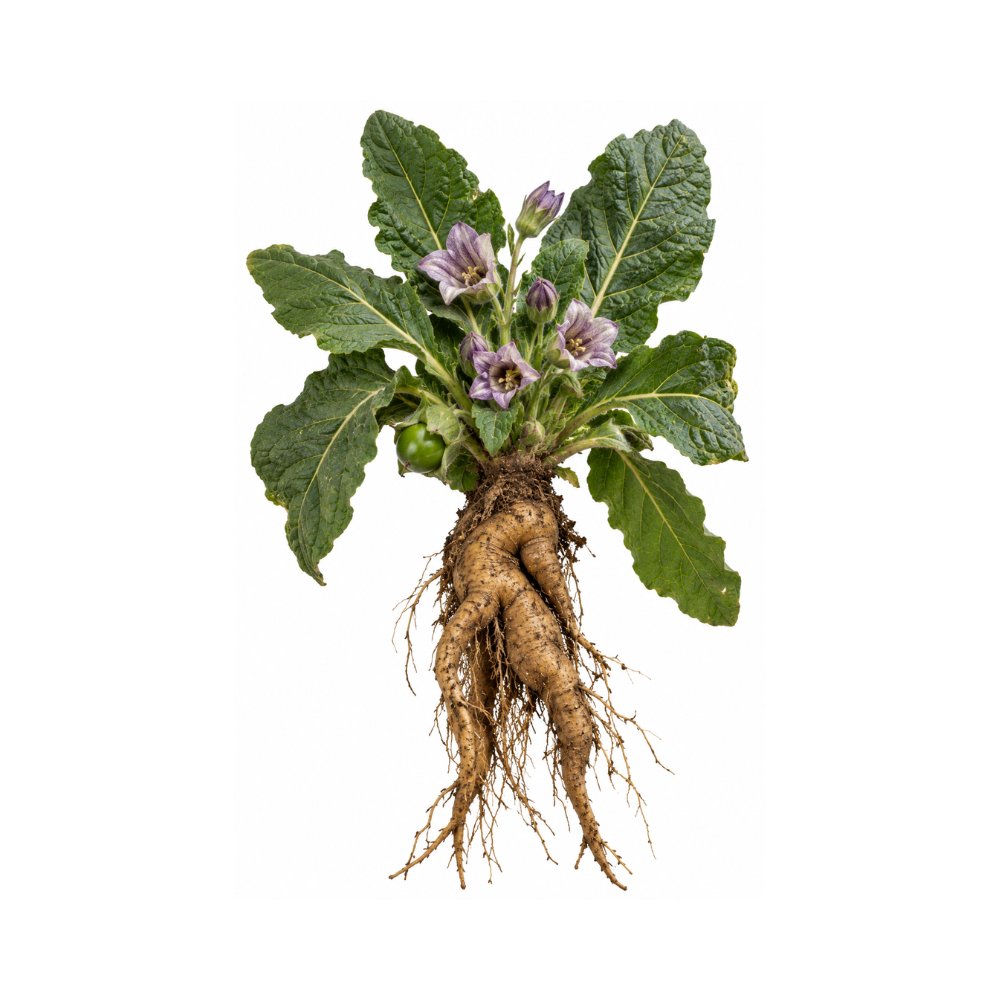 Source Mandrake ☠️ Mandragora officinarum Herb monograph →
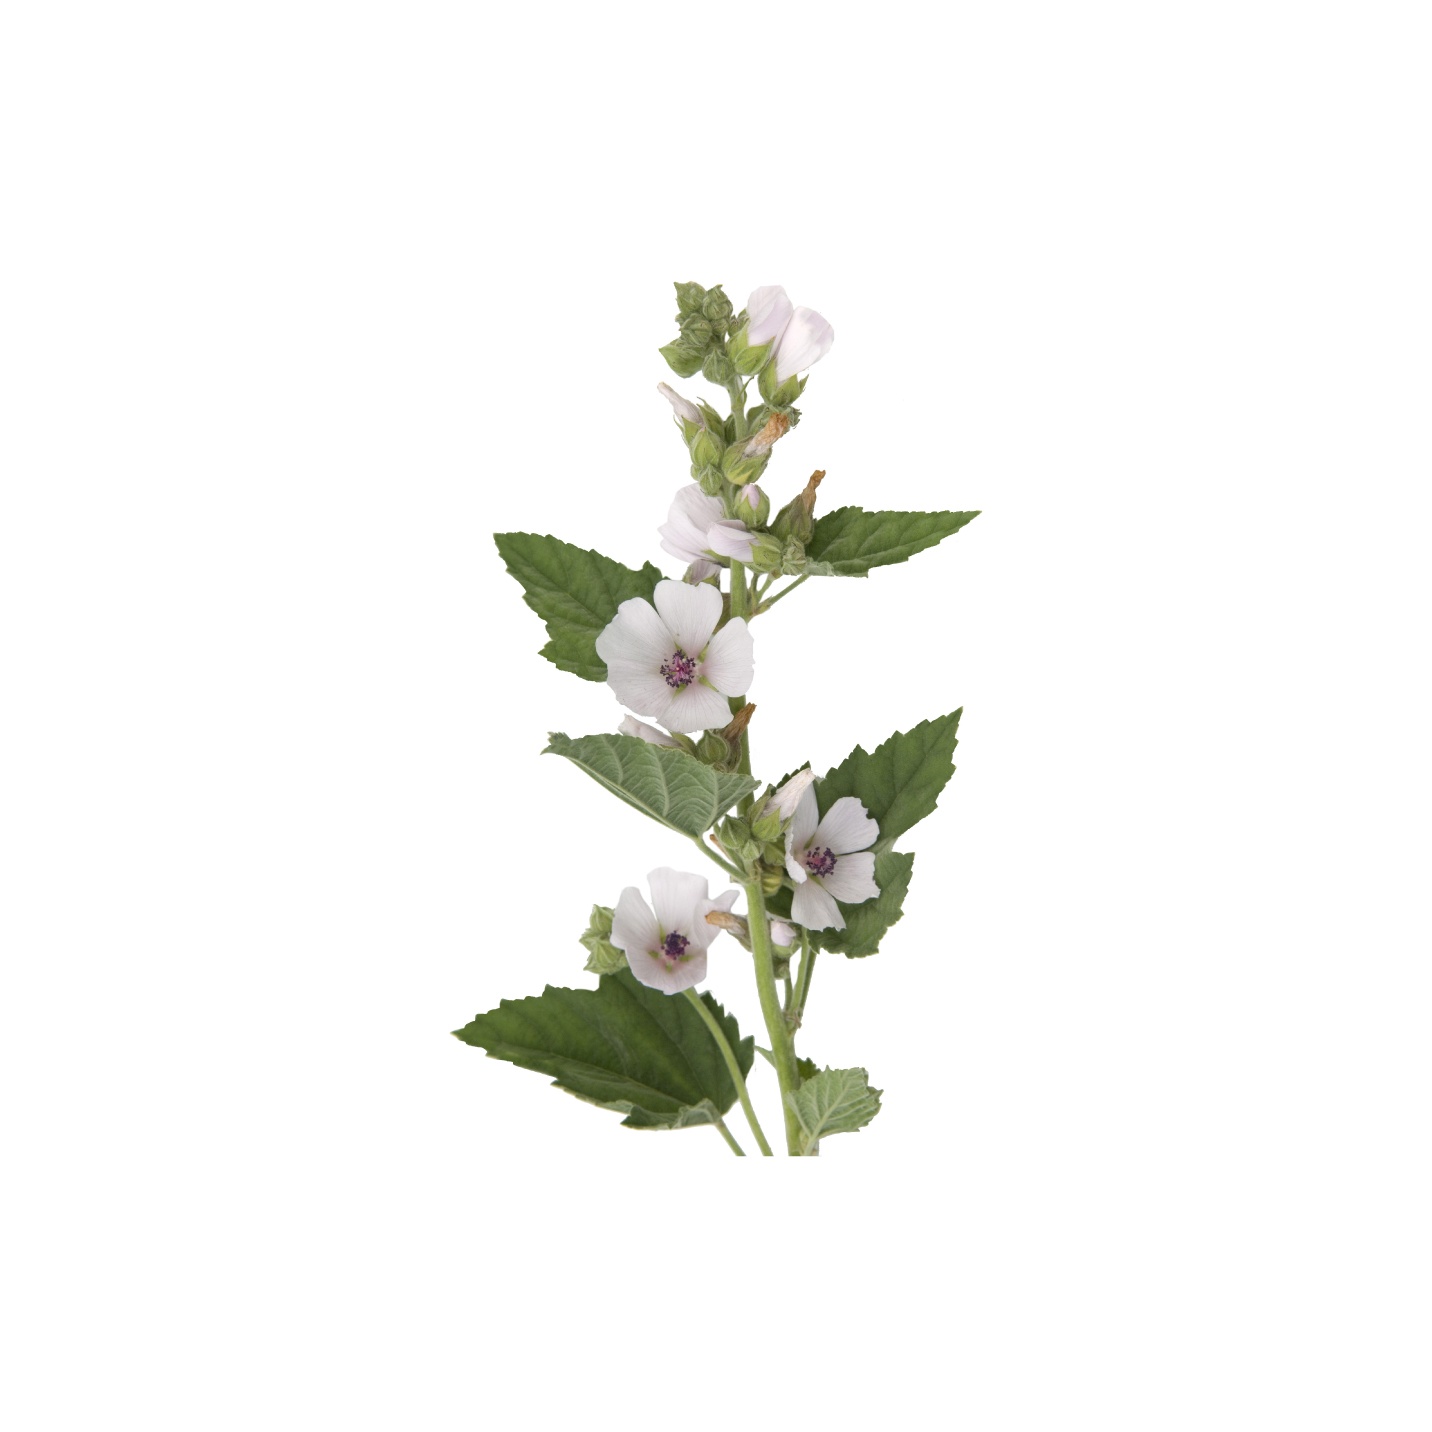 Source Marshmallow Althaea officinalis Herb monograph →
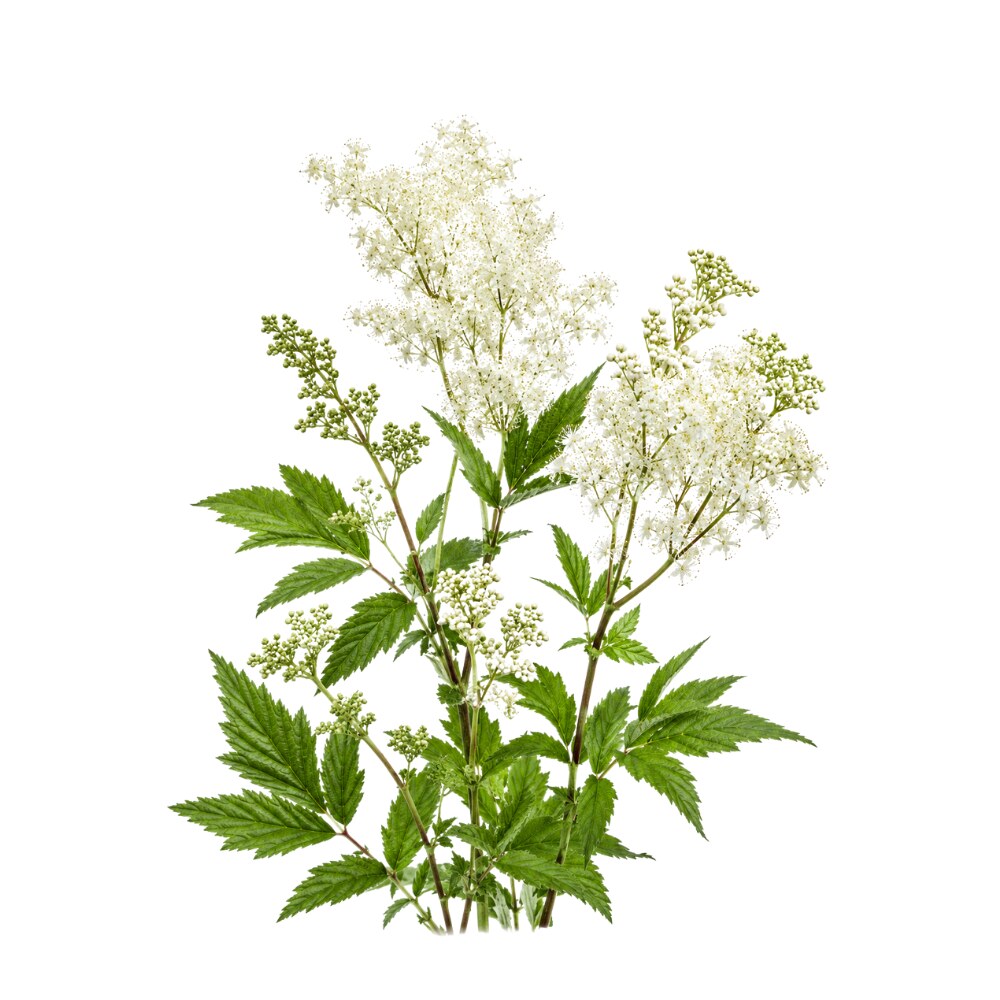 Source Meadowsweet Filipendula ulmaria Herb monograph →
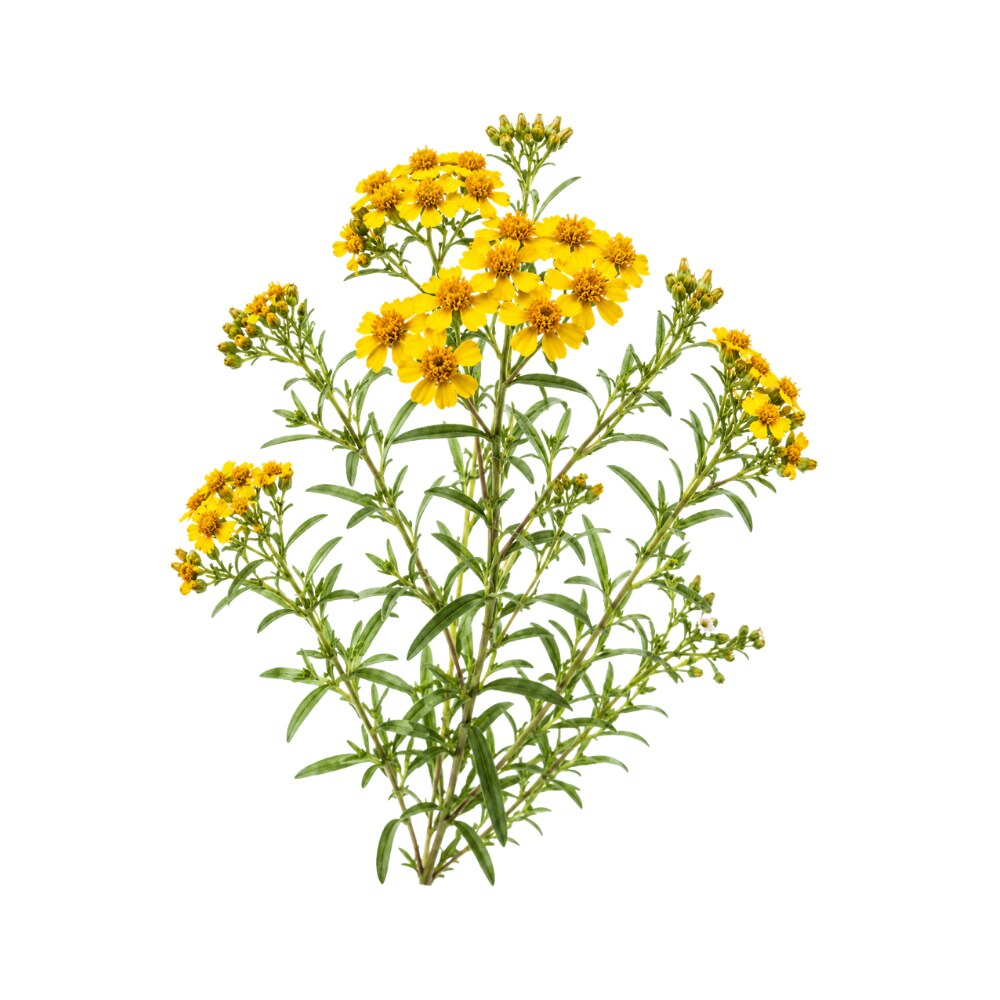 Source Mexican Tarragon Tagetes lucida Herb monograph →
 Source Mugwort Artemisia vulgaris Herb monograph →
 Source Passionflower Passiflora incarnata Herb monograph →
 Source Stevia Stevia rebaudiana Herb monograph →
 Source Sweet Wormwood Artemisia annua Herb monograph →
Concentration
Content by Source
Concentrations not reported. No percent-dry-weight or mg/g figures have been published for this compound in its source plants.
Scopoletin at a Glance
Scopoletin is a widely distributed plant hydroxycoumarin, found in noni, chicory, and many roots and barks.
Its preclinical research centres on anti-inflammatory activity through NF-kB and Nrf2, antioxidant effects, and xanthine-oxidase-mediated urate lowering — the last giving it a defined mechanism relevant to gout, in the same family as the xanthine oxidase inhibitors.
Scopoletin Is Not “Coumarin”
The single most common error about this molecule is a naming one, and it runs in both directions — inheriting a warning it does not deserve, and a reputation it has not earned.
Coumarin is the simple parent of the class: the bare benzopyranone of tonka bean and sweet woodruff, associated with dose-dependent hepatotoxicity and regulated in food. Warfarin and dicoumarol are 4-hydroxycoumarins, synthetic or fungal-fermentation products whose anticoagulant action comes from antagonising vitamin K epoxide reductase. Scopoletin is neither: it is a 6-methoxy-7-hydroxycoumarin, a simple hydroxy-methoxy substitution on the same skeleton, with no 4-hydroxy group and none of the chemistry that gives warfarin its action.
So the class-wide caution that “coumarins interact with blood thinners” overstates the risk here — vitamin-K-antagonist anticoagulation belongs to the 4-hydroxycoumarin subclass, not to scopoletin. And the hepatotoxicity concern attached to fragrance coumarin does not transfer either.
Its own near relatives are worth keeping straight for the same reason, since each has its own page and its own data:
- Scopolin — scopoletin’s glucoside, and a pro-drug form: it is hydrolysed back to scopoletin in vivo 15Reference 15AnimalEvaluation of the pharmacokinetics, bioavailability and urinary excretion of scopolin and its metabolite scopoletin in rats by LC-MS/MSView study →.
- Isoscopoletin — the 6-hydroxy-7-methoxy isomer, the same two groups the other way round.
- Scoparone — the 6,7-dimethoxy analogue.
- Umbelliferone — the plain 7-hydroxycoumarin, scopoletin’s biosynthetic sibling.
Scopoletin in Pelargonium — Present, But Not the Mechanism
Scopoletin is one of the characteristic root coumarins of Pelargonium sidoides and P. reniforme, the South African plants behind the respiratory-tract preparation EPs 7630, and its presence there is often read as an explanation for how that medicine works. The evidence in this species says otherwise, and the case is a clean worked example of a constituent being present without being responsible.
The antibacterial data are real but modest. In the study that isolated it from Pelargonium alongside umckalin, 5,6,7-trimethoxycoumarin and 6,8-dihydroxy-5,7-dimethoxycoumarin, scopoletin inhibited a panel of Gram-positive and Gram-negative bacteria at MICs of 200–1,000 µg/mL — the same band as the other active constituents, with (+)-catechin the only inactive one 18Reference 18In vitroAntibacterial activity of extracts and constituents of Pelargonium sidoides and Pelargonium reniforme — in vitroView study →. Those are weak concentrations by antibiotic standards.
The immunomodulatory activity is not the coumarins’. When the same group tested extracts and isolated constituents on non-specific immune function, the coumarin samples were the exception: every Pelargonium extract and both phenolic acids significantly reduced intracellular survival of Leishmania donovani amastigotes in macrophages — gallic acid at EC50 4.4 µg/mL and methyl gallate at 12.5 µg/mL — while the coumarins did not 19Reference 19In vitroImmunomodulatory principles of Pelargonium sidoides — in vitroView study →. The active immunomodulators were the phenolic acids.
And the anti-adhesive activity is not the coumarins’ either. EPs 7630’s ability to stop group A streptococci binding epithelial cells was traced to its proanthocyanidins, specifically the prodelphinidin type: polyphenol-free samples were inactive, and pre-treating the bacteria rather than the cells was what produced the effect 20Reference 20In vitroEvaluation of an aqueous-ethanolic extract from Pelargonium sidoides (EPs 7630) for its activity against group A-streptococci adhesion to human HEp-2 epithelial cells — in vitroView study →.
The honest summary is that scopoletin is a genuine and characteristic constituent of Pelargonium root, contributes a share of a modest antibacterial effect, and is not the reason the extract does what it does. Treat any claim that routes EPs 7630’s clinical evidence through this molecule as unsupported.
What It's Used For
Scopoletin’s pharmacology is entirely preclinical — there are no human trials of the isolate in any indication. Its best-defined activities are anti-inflammatory NF-κB/Nrf2 signalling, direct antioxidant scavenging, and xanthine-oxidase inhibition with a uricosuric, urate-lowering effect 1,
Scopoletin suppresses NF-κB (IκBα–p65) signaling and pro-inflammatory cytokines while inducing the Keap1–Nrf2/HO-1 antioxidant response, shown in cerulein pancreatitis and lung injury 4Reference 4AnimalProtective effect of scopoletin against cerulein-induced acute pancreatitis and associated lung injury in miceView study → and vancomycin nephro-intoxication models 5Reference 5AnimalAmeliorative impacts of scopoletin against vancomycin-induced intoxication in rats through Keap1-Nrf2/HO-1 and IκBα-P65 NF-κB/P38 MAPK pathwaysView study →, and reviewed across its targets 3Reference 3Modulation of multiple cellular signalling pathways as targets for anti-inflammatory and anti-tumorigenesis action of scopoletinView study →.
Gap: all animal and cell, with no isolated-compound human data and model-specific effect sizes 3,
Scopoletin is a direct free-radical scavenger 2Reference 2Antioxidant properties of scopoletin isolated from Sinomenium acutumView study → and protects hepatocytes against palmitate- and bile-acid-induced death by reducing ER and oxidative stress 8Reference 8Scopoletin and umbelliferone protect hepatocytes against palmitate- and bile-acid-induced cell death by reducing ER stress and oxidative stressView study →.
Gap: foundational but non-specific chemistry shared by hydroxycoumarins, concentration-dependent, with no in-vivo human antioxidant readout 2Reference 2Antioxidant properties of scopoletin isolated from Sinomenium acutumView study →. (Scopoletin also shows screening-level antimicrobial activity — isolated from Mexican tarragon 14Reference 14Antifungal and antibacterial activities of Mexican tarragon (Tagetes lucida)View study →, and from Pelargonium sidoides root at MICs of 200–1,000 µg/mL against eight bacterial species 18Reference 18In vitroAntibacterial activity of extracts and constituents of Pelargonium sidoides and Pelargonium reniforme — in vitroView study → — but only in vitro, and at concentrations far above anything achievable systemically.)
The signature scopoletin activity: it inhibits xanthine oxidase and adds a uricosuric action, lowering urate in a dedicated study 1Reference 1Hypouricemic action of scopoletin arising from xanthine-oxidase inhibition and uricosuric activityView study →, with a micelle formulation reproducing the antihyperuricemic effect in hyperuricemic mice 7Reference 7AnimalAntihyperuricemic efficacy of scopoletin-loaded Soluplus micelles in hyperuricemic miceView study →.
Gap: rodent only, with potency modest versus allopurinol/febuxostat and no clinical urate-lowering data — and the micelle requirement itself signals the free compound’s bioavailability limits 7Reference 7AnimalAntihyperuricemic efficacy of scopoletin-loaded Soluplus micelles in hyperuricemic miceView study →.
Scopoletin modulates monoamine oxidase A/B and brain monoamine levels 9Reference 9Effect of scopoletin on monoamine oxidases and brain aminesView study → and features among MAO-inhibitory coumarins 10Reference 10Coumarins with monoamine-oxidase inhibitory activity and antioxidative coumarino-lignans from Hibiscus syriacusView study →; it reduced anxiety-like behavior in an inflammatory-pain mouse model 6Reference 6AnimalScopoletin ameliorates anxiety-like behaviours in a complete-Freund’s-adjuvant-induced mouse modelView study →, within a broader picture of coumarin antidepressant activity 11Reference 11Antidepressant effects of coumarins and their derivatives: a critical analysis of research advancesView study →.
Gap: the behavioral antidepressant efficacy is mostly demonstrated for plant/coumarin fractions, not the purified isolate, and the MAO effects are moderate 9Reference 9Effect of scopoletin on monoamine oxidases and brain aminesView study →.
Scopoletin produced acute and chronic antihypertensive effects in rats in a single plant-isolate study 12Reference 12Acute and chronic antihypertensive effect of fractions, tiliroside and scopoletin from Malva parvifloraView study →.
Gap: one study, with the vasorelaxant mechanism inferred and not replicated for the isolate alone 12Reference 12Acute and chronic antihypertensive effect of fractions, tiliroside and scopoletin from Malva parvifloraView study →.
Scopoletin shows pro-apoptotic and autophagy-activating signals in tumor cells 3Reference 3Modulation of multiple cellular signalling pathways as targets for anti-inflammatory and anti-tumorigenesis action of scopoletinView study →, though the strongest anticancer data are for synthetic 3-aryl-7-hydroxy scopoletin derivatives, not native scopoletin 13Reference 13Design, synthesis and biological evaluation of 3-aryl-7-hydroxy scopoletin derivatives as autophagy activators against tumorigenesisView study →.
Gap: in-vitro-dominant and derivative-driven, with weak evidence for the parent compound 13Reference 13Design, synthesis and biological evaluation of 3-aryl-7-hydroxy scopoletin derivatives as autophagy activators against tumorigenesisView study →.
Mechanisms
| Target / pathway | Effect | Relevant to |
|---|---|---|
| Xanthine oxidase (inhibition) + renal urate handling | ↓ urate production + ↑ excretion | anti-hyperuricemia / gout |
| NF-κB (IκBα–p65) | ↓ pro-inflammatory cytokines | anti-inflammatory |
| Keap1–Nrf2 / HO-1 | ↑ antioxidant/cytoprotective response | antioxidantorgan protection |
| Direct ROS/radical scavenging | ↓ oxidative stress | antioxidant |
| Monoamine oxidase A/B (modulation) | ↑ brain monoamines | neuro / antidepressant |
Pharmacokinetics
Load-bearing and honestly limited. Scopoletin is a small hydroxy-methoxycoumarin with moderate-to-poor oral bioavailability — rapidly absorbed but extensively metabolized by phase-II conjugation (glucuronidation/sulfation, the coumarin-class pattern), giving short systemic exposure. Its glucoside scopolin is hydrolyzed to scopoletin in vivo, and both are cleared rapidly and excreted in urine 15Reference 15AnimalEvaluation of the pharmacokinetics, bioavailability and urinary excretion of scopolin and its metabolite scopoletin in rats by LC-MS/MSView study →; elimination from a standardized plant fraction likewise shows fast clearance 16Reference 16Elimination pharmacokinetics of a scopoletin-containing standardised fraction of Sphaeralcea angustifolia administered orallyView study →, and metabolite profiling documents the coumarin phase-I/II routes 17Reference 17Metabolic profiling of coumarins by UPLC-MS-based metabolomics and multiple mass-defect filterView study →. The fact that a micelle formulation was needed to achieve an antihyperuricemic effect in vivo 7Reference 7AnimalAntihyperuricemic efficacy of scopoletin-loaded Soluplus micelles in hyperuricemic miceView study → independently confirms real bioavailability constraints — this is not a well-absorbed oral agent. A validated HPLC-fluorescence assay for scopoletin in rat plasma, sensitive from 1 ng/mL, was published in 2024 and applied to a rat pharmacokinetic study — the analytical groundwork a proper exposure profile would need, and a marker of how little of that groundwork existed until recently 24Reference 24AnimalA simple and sensitive high-performance liquid chromatographic method combined with fluorescence detection for bioanalysis of scopoletin in rat plasma: application to a pharmacokinetic study — animal modelView study →.
Clinical Trials
There are no human trials of the isolated molecule for any indication. Human exposure occurs only via whole plants and products (noni juice, nettle, marshmallow), where scopoletin is one of many constituents and its individual contribution is not isolated — so any “clinical” framing belongs to the plant product, not the compound.
| Completed | Planned | Terminated | Preclinical |
|---|---|---|---|
| —(isolate); plant-product only | — | — | Extensive |
Last checked: July 2026.
Isolate vs. Plant Studies
The split is unusually clean, and it is the reason this molecule’s reputation runs ahead of its evidence.
Every pharmacological result above is isolate work — purified scopoletin in rodents or in cell culture 1,
But every human exposure is plant exposure, and in every plant scopoletin is a trace constituent among many. Noni juice, nettle, marshmallow, cleavers and Mexican tarragon each carry it at levels that no study has shown to reach a pharmacologically active plasma concentration — and the bioavailability data give a positive reason to doubt they do. Where a whole-plant preparation has been shown to work, the activity has repeatedly been traced to something else: in Pelargonium sidoides the immunomodulation belongs to the phenolic acids 19Reference 19In vitroImmunomodulatory principles of Pelargonium sidoides — in vitroView study → and the anti-adhesion to the prodelphinidins 20Reference 20In vitroEvaluation of an aqueous-ethanolic extract from Pelargonium sidoides (EPs 7630) for its activity against group A-streptococci adhesion to human HEp-2 epithelial cells — in vitroView study →, with the coumarins comparatively inactive. Where the isolate has been tested inside a plant fraction, it has usually been one contributor of several — as in the Malva parviflora antihypertensive study, where scopoletin and tiliroside were tested alongside the fractions rather than instead of them 12Reference 12Acute and chronic antihypertensive effect of fractions, tiliroside and scopoletin from Malva parvifloraView study →.
The honest position is that scopoletin is a well-characterised molecule with no demonstrated contribution to the effect of any herb that contains it.
Its Role in Plants
Scopoletin is not an incidental metabolite. In plants it is an inducible defence compound and an iron-acquisition tool, and both roles are unusually well worked out.
As a phytoalexin. In wild tobacco (Nicotiana attenuata), infection with the necrotrophic fungus Alternaria alternata triggers a blue fluorescence in leaves that was shown, by silencing the biosynthetic gene feruloyl-CoA 6′-hydroxylase 1 (F6′H1), to come from scopoletin and its glucoside scopolin. Scopoletin was strongly antifungal against the pathogen in vitro and in planta, its induction depended on jasmonate signalling through the master regulator MYC2, and plants unable to make it — or unable to perceive jasmonate — were highly susceptible. Young leaves accumulate more of it than mature leaves, which is why they resist better 21Reference 21In vitroScopoletin is a phytoalexin against Alternaria alternata in wild tobacco dependent on jasmonate signalling — in vitroView study →. The same compound, transferred as a non-host defence metabolite, protected soybean against Asian soybean rust 22Reference 22In vitroThe Arabidopsis non-host defence-associated coumarin scopoletin protects soybean from Asian soybean rust — in vitroView study →.
As an iron chelator. Arabidopsis roots secrete coumarins when iron is scarce, and scopoletin is the major one. It is the substrate for scopoletin 8-hydroxylase, encoded by a strongly iron-responsive gene, which converts it to fraxetin — the catechol-bearing coumarin that actually mobilises Fe(III) in alkaline soil 23Reference 23In vitroScopoletin 8-hydroxylase: a novel enzyme involved in coumarin biosynthesis and iron-deficiency responses in Arabidopsis — in vitroView study →. So scopoletin sits at a branch point: an antifungal end product in one direction, a precursor to an iron-scavenging siderophore-like molecule in the other. Its accumulation, and that of umbelliferone and their glycosides, varies substantially between natural Arabidopsis populations 26Reference 26In vitroGenes to specialized metabolites: accumulation of scopoletin, umbelliferone and their glycosides in natural populations of Arabidopsis thaliana — in vitroView study →.
These are plant-biology functions. A molecule’s job as a phytoalexin says nothing about what it does in a person — but it does explain why scopoletin turns up across so many unrelated families, and why its levels in a given plant sample depend on what that plant had recently been fighting.
Prevalence in Nature
Scopoletin is widely distributed and almost always minor. It is reported across the Solanaceae, Rubiaceae, Asteraceae, Apiaceae, Malvaceae, Brassicaceae, Urticaceae and Geraniaceae, among others — a distribution that reflects its position as a common branch off the general phenylpropanoid pathway rather than any taxonomic signature.
Within that spread, a few sources stand out for different reasons:
- Noni (Morinda citrifolia) — the best-known source, where scopoletin is used as a marker compound for standardising juice products.
- Root and bark tissue generally — cleavers, marshmallow, nettle, cramp bark, chicory and Pelargonium sidoides root 18Reference 18In vitroAntibacterial activity of extracts and constituents of Pelargonium sidoides and Pelargonium reniforme — in vitroView study →.
- Mexican tarragon (Tagetes lucida), from which it has been isolated with antifungal and antibacterial screening data 14Reference 14Antifungal and antibacterial activities of Mexican tarragon (Tagetes lucida)View study →.
- Tobacco and Arabidopsis, where content is inducible rather than fixed — rising sharply on fungal challenge or iron deficiency 21,
23Reference 21In vitroScopoletin is a phytoalexin against Alternaria alternata in wild tobacco dependent on jasmonate signalling — in vitroView study →Reference 23In vitroScopoletin 8-hydroxylase: a novel enzyme involved in coumarin biosynthesis and iron-deficiency responses in Arabidopsis — in vitroView study → .
That inducibility is the reason quantitative figures for scopoletin content are so inconsistent between studies, and why no per-source comparison can usefully be drawn: in several of its best-studied hosts the concentration is a function of the plant’s recent conditions rather than a stable property of the species. In none of them is it a major component of the biomass.
Discovery & Synthesis
Scopoletin takes its name from Scopolia, the Solanaceous genus it was obtained from; the original isolation report predates the indexed literature and no date or discoverer is asserted here rather than a guessed one. It is also encountered as chrysatropic acid, gelseminic acid and β-methylaesculetin in older sources — three names for the same molecule, worth recognising when reading nineteenth- and early-twentieth-century phytochemistry.
Biosynthesis is the well-mapped part. Scopoletin is made from the general phenylpropanoid pathway by ortho-hydroxylation of feruloyl-CoA, catalysed by the 2-oxoglutarate-dependent dioxygenase feruloyl-CoA 6′-hydroxylase (F6′H1), followed by trans/cis isomerisation and spontaneous lactonisation to close the coumarin ring 21Reference 21In vitroScopoletin is a phytoalexin against Alternaria alternata in wild tobacco dependent on jasmonate signalling — in vitroView study →. Glucosylation gives scopolin, the storage form. Downstream, scopoletin 8-hydroxylase converts it to fraxetin 23Reference 23In vitroScopoletin 8-hydroxylase: a novel enzyme involved in coumarin biosynthesis and iron-deficiency responses in Arabidopsis — in vitroView study →.
That pathway is now a metabolic-engineering target rather than a supply route: overexpressing the scopoletin biosynthetic pathway in poplar incorporated the coumarin into lignin and improved the processing of lignocellulosic biomass 25Reference 25In vitroOverexpression of the scopoletin biosynthetic pathway enhances lignocellulosic biomass processing — in vitroView study →. Scopoletin itself is a cheap, commercially available fine chemical — supplied synthetically or extracted from plant material for analytical use — and there is no meaningful extraction industry built on it.
Patents: not yet researched (future patent-loop pass).
Toxicity & Safety
Scopoletin looks benign in preclinical work, and the coumarin scare it inherits is a case of mistaken identity — it is neither the hepatotoxic fragrance coumarin nor a warfarin-type anticoagulant. The genuine cautions that remain are theoretical.
- Low-toxicity preclinical profile. It behaves as a protective antioxidant agent in organ-injury models, and occurs at trace levels in foods and common herbs.
- Not the coumarin you are thinking of. Not the hepatotoxic fragrance parent, and not a warfarin-type anticoagulant — the “coumarins interact with blood thinners” caution overstates the risk here.
- Avoid concentrated or supplemental use in pregnancy and lactation. No reproductive-toxicology study of the isolate exists.
- Theoretical urate-drug overlap. Possible additive xanthine-oxidase effects alongside urate-lowering medication.
- MAO modulation is a plausibility flag. Not demonstrated at dietary exposure.
Full Safety & Interactions Detail
Scopoletin has a low-toxicity preclinical profile: it behaves as a protective, antioxidant agent in the organ-injury models rather than a toxicant, and it occurs at trace levels in foods and common herbs. The class confusion that gives it a borrowed warning is a naming problem rather than a pharmacological one, and is set out in full above. Genuine interactions are only theoretical: possible additive xanthine-oxidase effects with urate-lowering drugs, and MAO modulation as a plausibility flag not demonstrated at dietary exposure. What is missing is more consequential than what is present — there is no repeat-dose toxicity study, no genotoxicity package and no human safety data for isolated scopoletin, so the low flag reflects trace exposure and an absence of signals rather than a demonstrated safety margin.
Dosage
There is no established human dose, and nothing here is a recommendation. Preclinical models used oral rodent doses of roughly 1–50 mg/kg/day across the anti-inflammatory, antioxidant, antihypertensive and antihyperuricemic studies, with in-vitro work at low-micromolar concentrations — figures that do not translate to a human dose, and which the bioavailability limits above make an inefficient basis for free-compound oral dosing.
References
- Ding Z, Dai Y, Wang Z (2005). Hypouricemic action of scopoletin arising from xanthine-oxidase inhibition and uricosuric activity. Planta Medica. https://pubmed.ncbi.nlm.nih.gov/15729630/
- Shaw CY, Chen CH, Hsu CC, et al. (2003). Antioxidant properties of scopoletin isolated from Sinomenium acutum. Phytotherapy Research. https://pubmed.ncbi.nlm.nih.gov/12916088/
- Sakthivel KM, Vishnupriya S, Priya Dharshini LC, et al. (2022). Modulation of multiple cellular signalling pathways as targets for anti-inflammatory and anti-tumorigenesis action of scopoletin. Journal of Pharmacy and Pharmacology. https://pubmed.ncbi.nlm.nih.gov/33847360/
- Leema G, Tamizhselvi R (2018). Protective effect of scopoletin against cerulein-induced acute pancreatitis and associated lung injury in mice. Pancreas. https://pubmed.ncbi.nlm.nih.gov/29595543/
- Khalaf MM, Hassan SM, Sayed AM, et al. (2022). Ameliorative impacts of scopoletin against vancomycin-induced intoxication in rats through Keap1-Nrf2/HO-1 and IκBα-P65 NF-κB/P38 MAPK pathways. International Immunopharmacology. https://pubmed.ncbi.nlm.nih.gov/34848155/
- Luo L, Sun T, Yang L, et al. (2020). Scopoletin ameliorates anxiety-like behaviours in a complete-Freund’s-adjuvant-induced mouse model. Molecular Brain. https://pubmed.ncbi.nlm.nih.gov/32019580/
- Zeng Y, Ma Y, Yang Z, et al. (2020). Antihyperuricemic efficacy of scopoletin-loaded Soluplus micelles in hyperuricemic mice. Drug Development and Industrial Pharmacy. https://pubmed.ncbi.nlm.nih.gov/32811191/
- Wu Z, Geng Y, Buist-Homan M, et al. (2022). Scopoletin and umbelliferone protect hepatocytes against palmitate- and bile-acid-induced cell death by reducing ER stress and oxidative stress. Toxicology and Applied Pharmacology. https://pubmed.ncbi.nlm.nih.gov/34979142/
- Basu M, Mayana K, Xavier S, et al. (2016). Effect of scopoletin on monoamine oxidases and brain amines. Neurochemistry International. https://pubmed.ncbi.nlm.nih.gov/26796202/
- Yun BS, Lee IK, Ryoo IJ, et al. (2001). Coumarins with monoamine-oxidase inhibitory activity and antioxidative coumarino-lignans from Hibiscus syriacus. Journal of Natural Products. https://pubmed.ncbi.nlm.nih.gov/11575966/
- Akwu NA, Lekhooa M, Deqiang D, et al. (2023). Antidepressant effects of coumarins and their derivatives: a critical analysis of research advances. European Journal of Pharmacology. https://pubmed.ncbi.nlm.nih.gov/37543158/
- Lagunas-Herrera H, Tortoriello J, Herrera-Ruiz M, et al. (2019). Acute and chronic antihypertensive effect of fractions, tiliroside and scopoletin from Malva parviflora. Biological & Pharmaceutical Bulletin. https://pubmed.ncbi.nlm.nih.gov/30606987/
- Lu X, Zhu C, Zhang C, et al. (2022). Design, synthesis and biological evaluation of 3-aryl-7-hydroxy scopoletin derivatives as autophagy activators against tumorigenesis. European Journal of Medicinal Chemistry. https://pubmed.ncbi.nlm.nih.gov/36242987/
- Céspedes CL, et al. (2006). Antifungal and antibacterial activities of Mexican tarragon (Tagetes lucida). Journal of Agricultural and Food Chemistry. https://pubmed.ncbi.nlm.nih.gov/19127719/
- Li B, Lu M, Chu Z, et al. (2019). Evaluation of the pharmacokinetics, bioavailability and urinary excretion of scopolin and its metabolite scopoletin in rats by LC-MS/MS. Biomedical Chromatography. https://pubmed.ncbi.nlm.nih.gov/31412148/
- Serrano-Román J, Nicasio-Torres P, Hernández-Pérez E, et al. (2020). Elimination pharmacokinetics of a scopoletin-containing standardised fraction of Sphaeralcea angustifolia administered orally. Journal of Pharmaceutical and Biomedical Analysis. https://pubmed.ncbi.nlm.nih.gov/32045824/
- Xiao Y, Wang YK, Xiao XR, et al. (2020). Metabolic profiling of coumarins by UPLC-MS-based metabolomics and multiple mass-defect filter. Xenobiotica. https://pubmed.ncbi.nlm.nih.gov/32174209/
- Kayser O, Kolodziej H (1997). Antibacterial activity of extracts and constituents of Pelargonium sidoides and Pelargonium reniforme — in vitro. Planta Medica. https://pubmed.ncbi.nlm.nih.gov/9434601/
- Kayser O, Kolodziej H, Kiderlen AF (2001). Immunomodulatory principles of Pelargonium sidoides — in vitro. Phytotherapy Research. https://doi.org/10.1002/ptr.785
- Janecki A, Conrad A, Engels I, et al. (2011). Evaluation of an aqueous-ethanolic extract from Pelargonium sidoides (EPs 7630) for its activity against group A-streptococci adhesion to human HEp-2 epithelial cells — in vitro. Journal of Ethnopharmacology. https://pubmed.ncbi.nlm.nih.gov/20883767/
- Sun H, Wang L, Zhang B, et al. (2014). Scopoletin is a phytoalexin against Alternaria alternata in wild tobacco dependent on jasmonate signalling — in vitro. Journal of Experimental Botany. https://pubmed.ncbi.nlm.nih.gov/24821958/
- Beyer SF, Beesley A, Rohmann PFW, et al. (2019). The Arabidopsis non-host defence-associated coumarin scopoletin protects soybean from Asian soybean rust — in vitro. The Plant Journal. https://pubmed.ncbi.nlm.nih.gov/31148306/
- Siwinska J, Siatkowska K, Olry A, et al. (2018). Scopoletin 8-hydroxylase: a novel enzyme involved in coumarin biosynthesis and iron-deficiency responses in Arabidopsis — in vitro. Journal of Experimental Botany. https://pubmed.ncbi.nlm.nih.gov/29361149/
- Kim T, Han DG, Yoon IS (2024). A simple and sensitive high-performance liquid chromatographic method combined with fluorescence detection for bioanalysis of scopoletin in rat plasma: application to a pharmacokinetic study — animal model. Biomedical Chromatography. https://pubmed.ncbi.nlm.nih.gov/39039810/
- Hoengenaert L, Wouters M, Kim H, et al. (2022). Overexpression of the scopoletin biosynthetic pathway enhances lignocellulosic biomass processing — in vitro. Science Advances. https://pubmed.ncbi.nlm.nih.gov/35857515/
- Ihnatowicz A, Siwinska J, Perkowska I, et al. (2024). Genes to specialized metabolites: accumulation of scopoletin, umbelliferone and their glycosides in natural populations of Arabidopsis thaliana — in vitro. BMC Plant Biology. https://pubmed.ncbi.nlm.nih.gov/39187756/



